 |
LandscapeDNDC 1.37.0
|
|
LandscapeDNDC 1.37.0
|

MeTrx simulates carbon and nitrogen cycle of soils. Focus lies on the production and consumption of the greenhouse gases \( CO_2, CH_4 \) and \( N_2O \). Therewith related outputs include leaching of \( NO_3 \) and emissions of \( NH_3 \). Depending on the ecosystem of interest, several model options should be considered (see also: metrxoptions):
Microbial processes are especially relevant in the upper soil layers. Choose a spatial discretization of at maximum 0.5 cm for the upper 1cm soil depth. For a soil depth greater 1cm and smaller 10 cm, a spatal discretization of 1-2 cm per soil layer is recommended.
MeTrx requires further models for:
MeTrx includes the following siteparameters:
The calibration of nitrogen trace gas emissions primarily addresses microbial metabolism, anaerobic conditions, and transport. The processes of decomposition and humification of SOM should be excluded or managed carefully in order to avoid compromising the overall stability of SOM by inadvertently inducing unrealistically high losses or gains.
| name | mean | min | max | coderef | calibration_target |
|---|---|---|---|---|---|
| METRX_MUEMAX_C_MIC | 5 | 3 | 7 | Microbial dynamics | SOC |
| METRX_AMAX | 1 | 0.5 | 1.5 | Microbial dynamics | N2O,SOC |
| METRX_F_MIC_T_EXP_1 | 3.5 | 2 | 5 | ? | N2O,SOC |
| METRX_F_MIC_T_EXP_2 | 35 | 25 | 40 | ? | N2O,SOC |
| METRX_F_MIC_M_WEIBULL_1 | 0.6 | 0.3 | 0.7 | Temperature and moisture dependency of microbial growth | SOC |
| METRX_F_MIC_M_WEIBULL_2 | 9 | 5 | 20 | Temperature and moisture dependency of microbial growth | SOC |
| name | mean | min | max | coderef | calibration_target |
|---|---|---|---|---|---|
| METRX_AMAX | 1 | 0.5 | 1.5 | Microbial dynamics | N2O,SOC |
| METRX_F_MIC_T_EXP_1 | 3.5 | 2 | 5 | ? | N2O,SOC |
| METRX_F_MIC_T_EXP_2 | 35 | 25 | 40 | ? | N2O,SOC |
| METRX_MUEMAX_C_DENIT | 0.5 | 0.2 | 2 | Denitrifier growth | N2O |
| METRX_KMM_C_DENIT | 0.005 | 0.0001 | 0.01 | Denitrifier growth | N2O |
| METRX_KMM_N_DENIT | 0.002 | 0.0001 | 0.01 | Denitrifier growth | N2O |
| METRX_F_DENIT_M_WEIBULL_1 | 0.85 | 0.4 | 0.95 | ? | N2O |
| METRX_F_DENIT_M_WEIBULL_2 | 25 | 6 | 30 | ? | N2O |
| METRX_F_DENIT_NO | 14 | 8 | 20 | ? | N2O |
| METRX_F_DENIT_N2_1 | 0.7 | 0 | 1 | ? | N2O |
| METRX_F_DENIT_N2_2 | 0.85 | 0.2 | 0.9 | ? | N2O |
| METRX_F_DENIT_PH_1 | 4.3 | 3 | 5.5 | ? | N2O |
| METRX_F_DENIT_PH_2 | 0.9 | 0.3 | 1.5 | ? | N2O |
| METRX_F_DENIT_N2O_PH_1 | 5 | 4 | 6.5 | ? | N2O |
| METRX_F_DENIT_N2O_PH_2 | 0.6 | 0.3 | 1.5 | ? | N2O |
| METRX_F_NIT_FRAC_MIC | 0.35 | 0.1 | 1 | NH4 nitrification | N2O |
| METRX_F_NIT_NO_N2O_T_EXP_1 | 0.033 | 0.01 | 0.1 | Production of NO and N2O during nitrification | N2O |
| METRX_F_NIT_NO_N2O_T_EXP_2 | 8.9 | 7 | 15 | Production of NO and N2O during nitrification | N2O |
| METRX_F_NIT_NO_N2O_M_WEIBULL_1 | 0.7 | 0.1 | 0.9 | Production of NO and N2O during nitrification | N2O |
| METRX_F_NIT_NO_N2O_M_WEIBULL_2 | 10 | 2 | 15 | Production of NO and N2O during nitrification | N2O |
| METRX_F_NIT_NO_M_EXP_1 | 8 | 2 | 15 | Production of NO and N2O during nitrification | N2O |
| METRX_F_NIT_NO_M_EXP_2 | 0.3 | 0 | 1 | Production of NO and N2O during nitrification | N2O |
| METRX_KMM_O2_NIT | 0.01 | 0.001 | 0.1 | NH4 nitrification | N2O |
| METRX_KMM_NH4_NIT | 0.001 | 1e-05 | 0.002 | NH4 nitrification | N2O |
| METRX_KMM_NO2_NIT | 5e-05 | 1e-05 | 0.001 | NO2 nitrification | N2O |
| METRX_KF_NIT_NO_N2O | 0.007 | 0.001 | 0.05 | Production of NO and N2O during nitrification | N2O |
| METRX_F_SANVF_1 | 2 | 1.6 | 3.5 | Anaerobic volume | N2O,NO |
| METRX_F_SANVF_2 | 7 | 6.3 | 15 | Anaerobic volume | N2O,NO |
| name | mean | min | max | coderef | calibration_target |
|---|---|---|---|---|---|
| METRX_F_SANVF_1 | 2 | 1.6 | 3.5 | Anaerobic volume | N2O,NO |
| METRX_F_SANVF_2 | 7 | 6.3 | 15 | Anaerobic volume | N2O,NO |
Available model options: Default options are marked with bold letters.
yes for agricultural rice production ecosystems for which growth of algae should be considered.Under construction.
MeTrx includes several model-specifc output options:
In order to include a MeTrx specific output, add the according attribute to the sinks section in the project file. Example:
The allocation of soil organic matter to various humus pools is primarily influenced by the C/N ratio within each pool, while adhering to the overall constraint of maintaining the soil's overarching C/N ratio.
The target C/N ratio of all mineral associated organic matter pools depend on the overall soil C/N ratio. Humus pool 1 representes non-protected organic matter. Humus pool 2 and 3 represent "old" and "very old" protected soil organic matter, respectively:
\begin{eqnarray*} C/N_{hum,1} &=& C/N_{soil} \\ C/N_{hum,2} &=& 1.5 \cdot C/N_{soil} \\ C/N_{hum,3} &=& METRX\_CN\_FRAC\_HUM3 \cdot C/N_{soil} \\ \end{eqnarray*}
Active organic material is assigned to microbial necromass (15%) and mineral associated but non-protected organic matter (humus pool 1: 85%).
Incoming litter from, e.g., plants, algae, animals is fragmentated to 'soil organic' litter (no more distinguishable from soil organic matter)
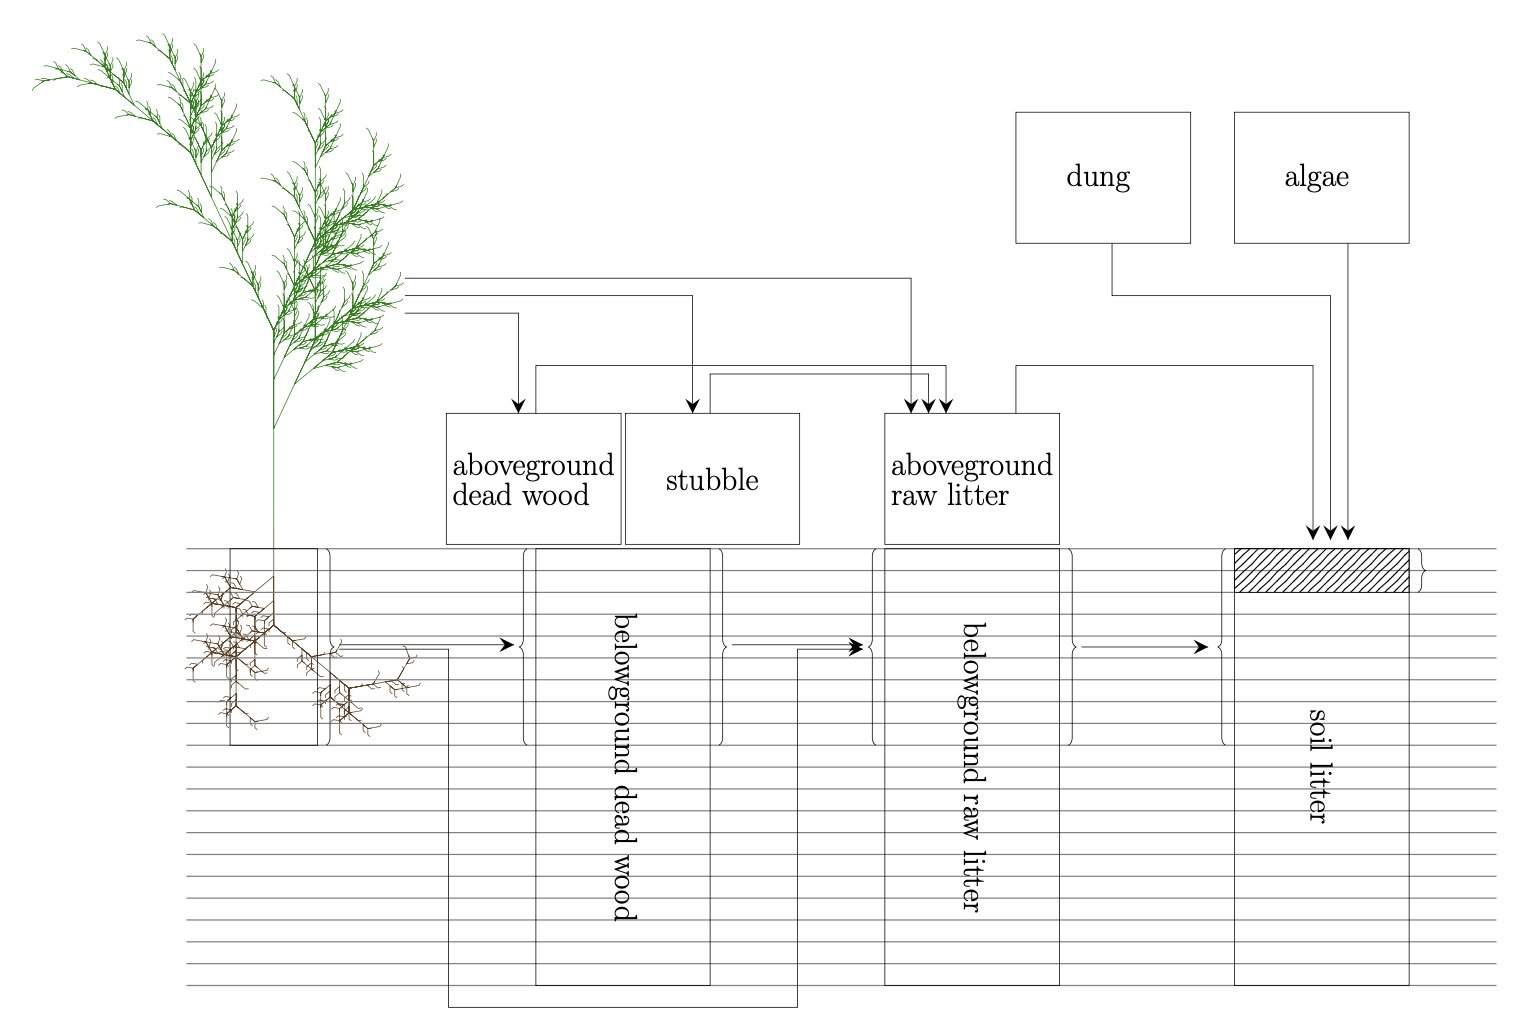
Turnover of soil organic matter (SOM) includes
Dissolved organic carbon is distinguished between the aerob and the anaerob soil and facilitates microbial metabolism (e.g., nitrification, denitrification, fermentation, ...). During fermentation and synthrophic metabolism, anaerob DOC can be further metabolized to acetate and molecular hydrogen, which serves methanogenic microbes as substrate. Decomposed nitrogen is always transferred to the dissolved organic nitrogen pool (DON) from where it is subsequently redistributed depending on pool specific target CN ratios.
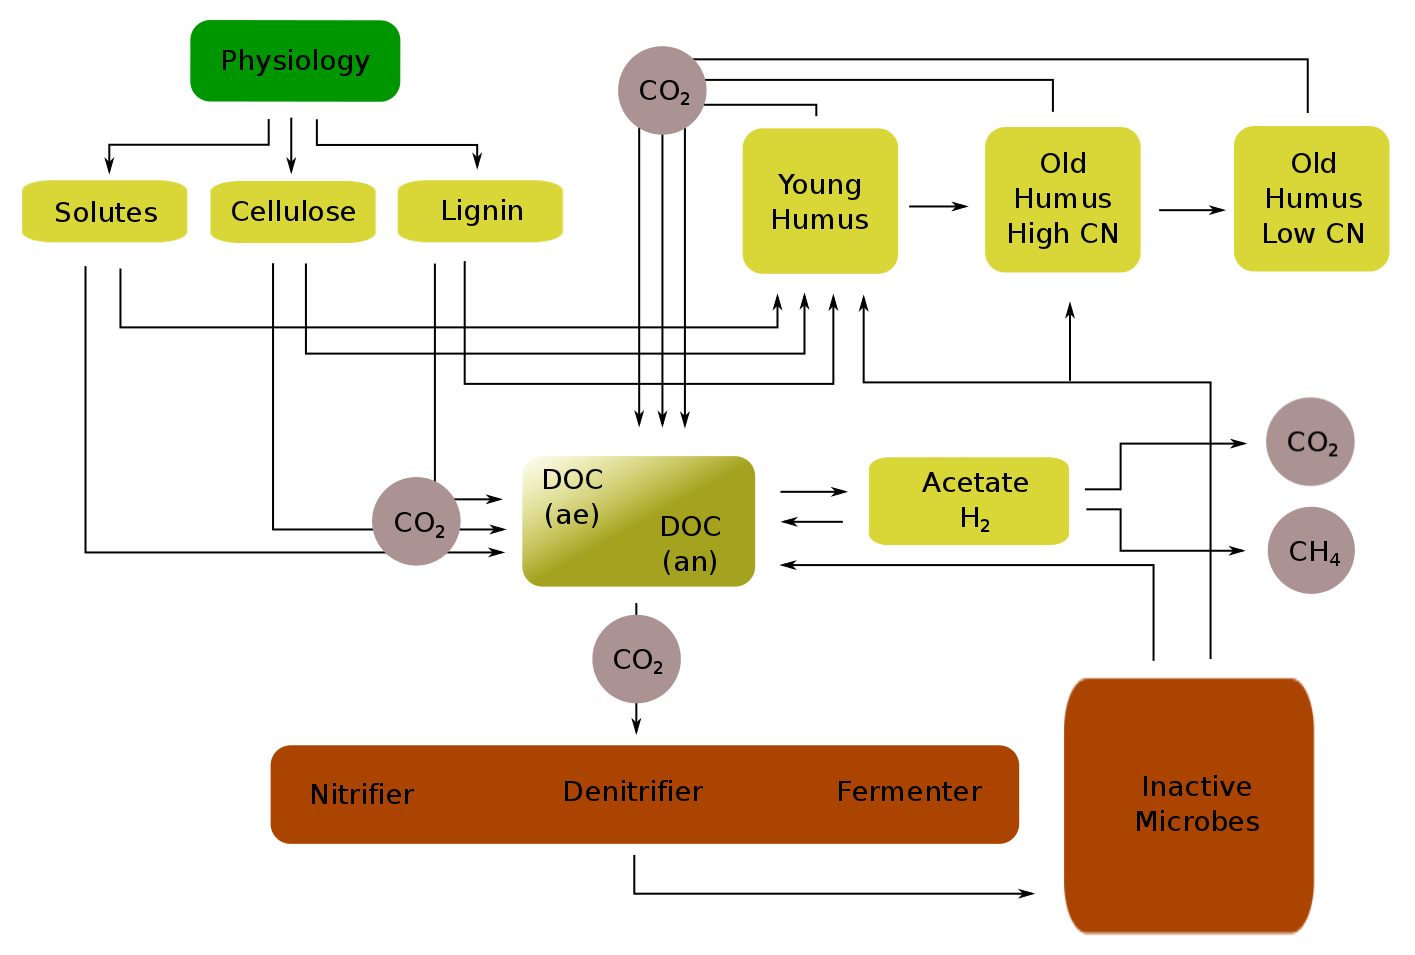
Turnover of microbial necromass involves:
Decomposition of inactive microbial carbon \( m_{imc} \) and nitrogen \( m_{imn} \) depends on soil temperature, soil moisture and soil anaerobicity:
\begin{eqnarray*}\Delta m_{imc \rightarrow doc_{ae}} = K\_DC\_AORG \cdot m_{imc} \cdot \phi_{tm} \cdot \phi_{till} \cdot (1 - anvf) \\ \Delta m_{imc \rightarrow doc_{an}} = K\_DC\_AORG \cdot m_{imc} \cdot \phi_{tm} \cdot \phi_{till} \cdot anvf \\ \Delta m_{imn} = \frac{\Delta m_{imc \rightarrow doc_{ae}} + \Delta m_{imc \rightarrow doc_{ae}}}{CN_{im}} \\ \end{eqnarray*}
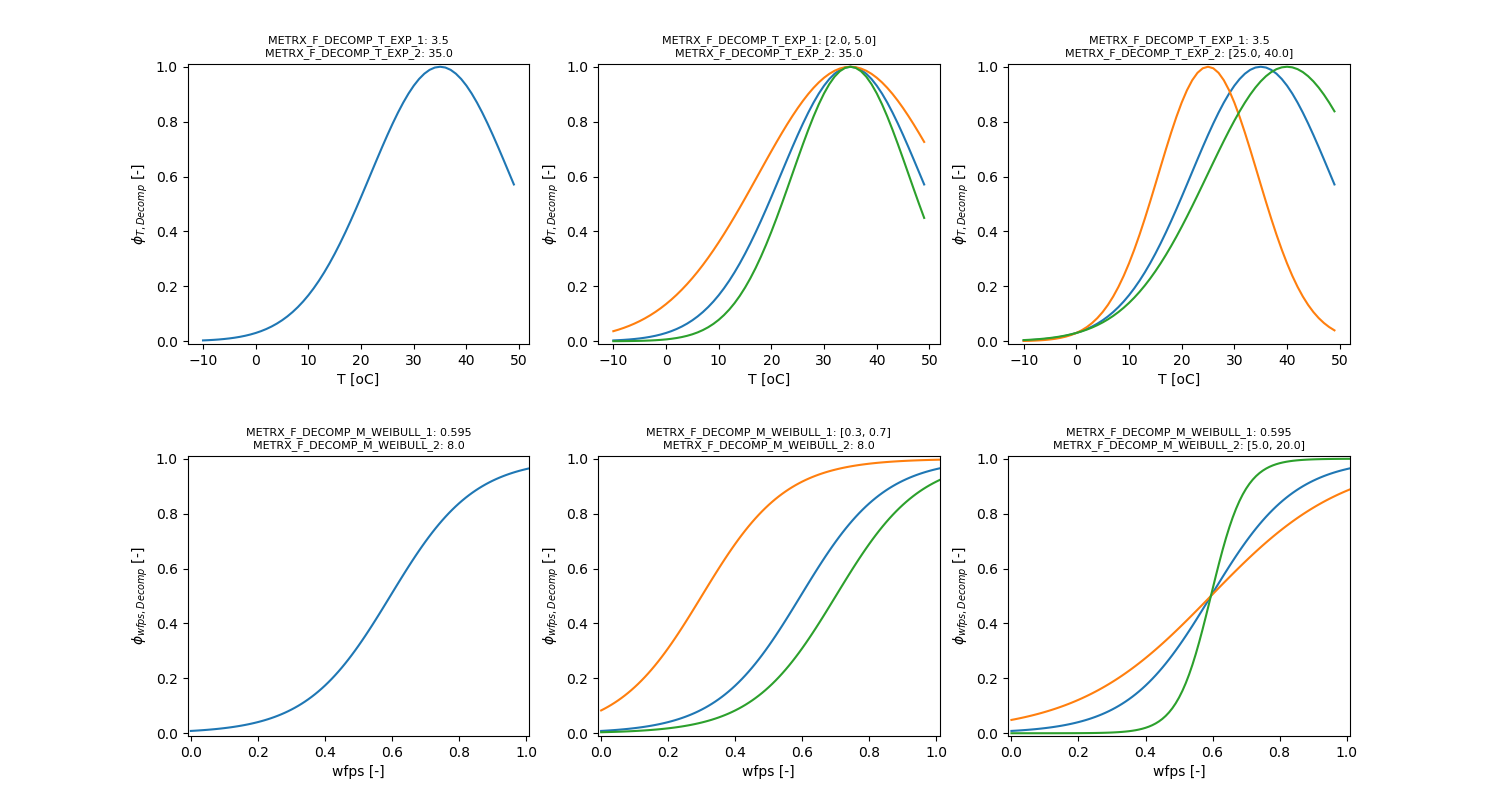
Temperature moisture factor
Humification of inactive microbial carbon is given by:
\begin{eqnarray*}\Delta m_{imc \rightarrow hum (young)} = METRX\_KR\_HU\_AORG\_HUM\_0 \cdot m_{imc} \\ \Delta m_{imc \rightarrow hum (old, high CN)} = METRX\_KR\_HU\_AORG\_HUM\_1 \cdot m_{imc} \\ \end{eqnarray*}
Turnover of SOM and plant debris includes:
Turnover rates depend on:
Depending on the litter or humus pool the general turnover rate is given by:
\[\frac{dm_x}{dt} = K_x \cdot m_x \cdot \Pi_i \phi_{i} \]
with \( \Pi_i \phi_{i} \) being the multiplicative combination of pool specific environmental reduction factors \( \phi_{i} \) (e.g., temperature, moisture,...) determining turnover.
The influence of temperature and moisture is given by:
\[\phi_{t,m} = \frac{2}{\frac{1}{\phi_{t}} + \frac{1}{\phi_{m}}} \]
The influence of the lignin content of the litter is given by:
\[\phi_{lig} = e^{-METRX\_BETA\_LITTER\_TYPE \cdot \frac{c_{lig}}{c_{tot}}} \]
The influence of litter quality (C/N ratio) is given by:
\[\phi_{litter} = 1 - METRX\_KR\_REDUCTION\_CN \cdot \frac{C_{lit}}{N_{lit}} \]
The influence of C/N ratio on anaerobic decomposition of humus pool 2 / organic soil
\[\phi_{cn,org. soil} = 1 - \frac{1}{1 + e^{-0.5 (C/N - 30}} \]
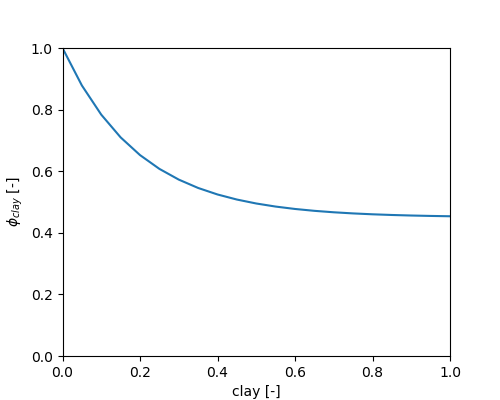
The influence of clay content is given by
\[\phi_{clay} = METRX\_F\_DECOMP\_CLAY\_1 + (1- METRX\_F\_DECOMP\_CLAY\_1) \cdot e^{-METRX\_F\_DECOMP\_CLAY\_2 \cdot c_{clay}} \]
The influence of O2 availability is given by the anaerobic volume fraction ( \( anvf \)). The carbon flux from each litter and humus pool due to decomposition is distinguished by \( anvf \):
\begin{eqnarray*}\frac{dm_x}{dt} &=& \frac{dm_{x, anvf}}{dt} + \frac{dm_{x, aevf}}{dt} \\ \frac{dm_{x, anvf}}{dt} &=& K_x \cdot m_x \cdot \Pi_j \phi_{j} \cdot METRX\_KR\_REDUCTION\_ANVF \cdot anvf \\ \frac{dm_{x, aevf}}{dt} &=& K_x \cdot m_x \cdot \Pi_j \phi_{j} \cdot (1 - \end{eqnarray*}
The influence of pH is given by:
\[\phi_{pH} = \frac{1}{1 + e^{-\frac{pH - \Omega_{MFDCP1}}{\Omega_{MFDCP2}}}} \]
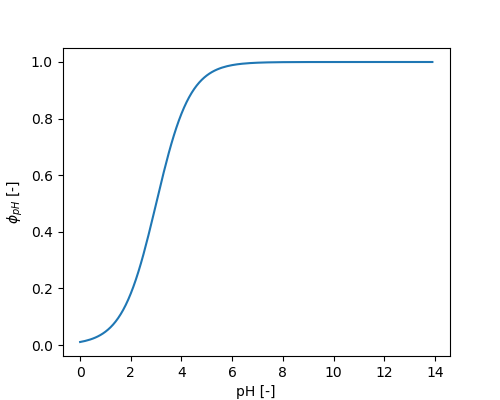
Overview of reduction factors for decomposition of litter and humus pools
| Pool | Parameter | tilling | Temp. Moisture | pH | litter type | litter C/N | clay | O2 |
|---|---|---|---|---|---|---|---|---|
| Solutes | METRX_KR_DC_SOL | yes | yes | yes | yes | yes | no | yes |
| Cellulose | METRX_KR_DC_CEL | yes | yes | yes | yes | yes | no | yes |
| Lignin | METRX_KR_DC_CEL | yes | yes | yes | yes | yes | no | yes |
| Humus 1 | METRX_KR_DC_HUM1 | yes | yes | yes | no | no | yes | yes |
| Humus 2 | METRX_KR_DC_HUM2 | yes | yes | yes | no | no | yes | yes |
| Humus 3 | METRX_KR_DC_HUM3 | yes | yes | yes | no | no | yes | yes |
Decomposed carbon is added to DOC:
\begin{eqnarray*}\frac{dDOC_{ae}}{dt} &=& -\frac{dC_{x, aevf}}{dt} \\ \frac{dDOC_{an}}{dt} &=& -\frac{dC_{x, anvf}}{dt} \end{eqnarray*}
Decomposed nitrogen is partly mineralized and partly added to DON:
\begin{eqnarray*}\frac{dNH_4}{dt} &=& -0.5 \frac{dN_{x}}{dt} \\ \frac{dDON}{dt} &=& -0.5 \frac{dN_{x}}{dt} \end{eqnarray*}
Microbial growth is given by:
\[\frac{c_{mic}}{dt} = c_{mic} \mu_{mic} \phi_{tm} \phi_{DOC} \]
Microbial activity \( \phi_{tm} \) is given a harmonic mean of a soil temperature ( \( \phi_{t}\)) and a soil water ( \( \phi_{m}\)) depending response coefficient.
\[\phi_{tm} = \frac{2}{\frac{1}{\phi_{t}} + \frac{1}{\phi_{m}}} \]
with \( \phi_{t}\) given by:
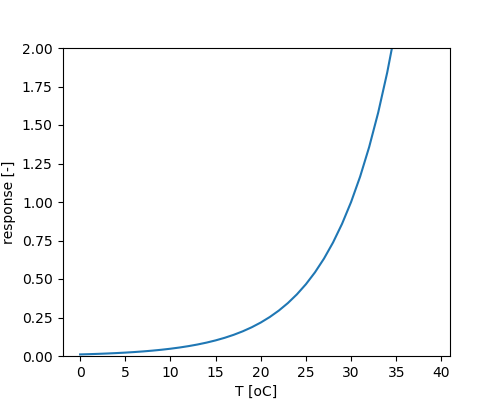
\[\phi_{t} = e^{-\Omega_{MFMTE1} \cdot \left( 1 - \frac{T}{\Omega_{MFMTE2}} \right)^2} \]
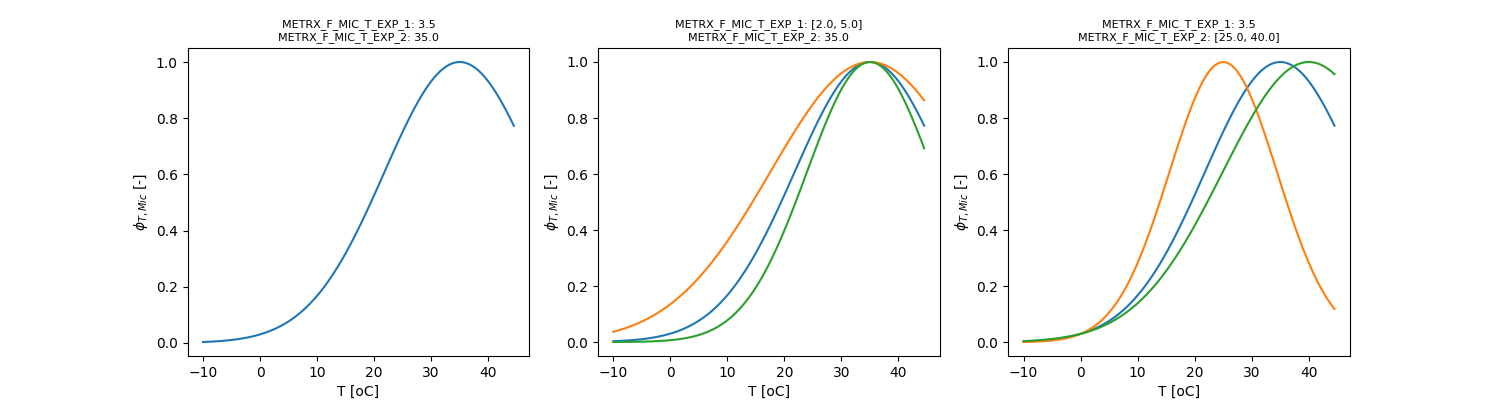
and with \( \phi_{m}\) given by a logistic function of the water content relative to field capacity ( \( \theta_{rel} = \theta / \theta_{fc} \), bounded to [0.001, 0.999]):
\[\phi_{m} = 1 - \frac{1}{1 + e^{(\theta_{rel} - \Omega_{MFMMW1}) \cdot \Omega_{MFMMW2}}} \]
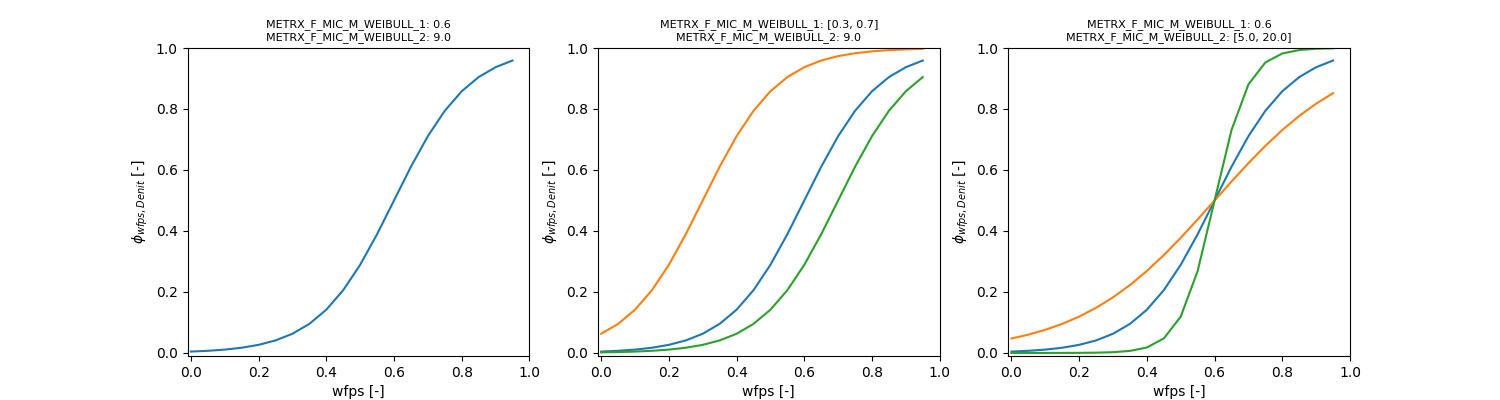
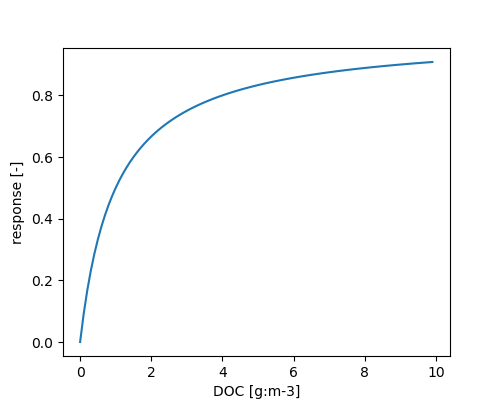
The dependency of microbial growth on DOC is given by:
\[\phi_{DOC} = \frac{DOC}{DOC + \Omega_{MKCM}} \]
Microbial loss of biomass via maintenance respiration \( \frac{c_{mic,r}}{dt} \) and death \( \frac{c_{mic,d}}{dt} \) are calculated after [7] :
\begin{eqnarray*}\frac{c_{mic,r}}{dt} &=& c_{mic} a_{mic} \phi_{tm} (1 - Y_r) \\ \frac{c_{mic,d}}{dt} &=& c_{mic} a_{mic} \phi_{tm} \phi_{C} \end{eqnarray*}
\( \phi_{tm}: \) Microbial activity
\[\phi_{C} = \frac{1}{1 + \Omega_{MKCM} \cdot DOC} \]
Nitrification is modeled as a two-stage process in the aerobic soil volume fraction \( V_{ae} = 1 - V_{an} \):
\[NH_4^+ \rightarrow NO_2^- \rightarrow NO_3^- \]
Nitrifiers are not represented as a separate microbial pool. Instead, a constant fraction of the aerobic microbial biomass \( C_{mic,1} \) is assumed to be able to nitrify. Carbon fixation by autotrophic nitrifiers is not considered.
The first step of nitrification (oxidation of \( NH_4^+ \) to \( NO_2^- \)) is given by:
\[N_{nit} = C_{nit} \, a_{mic} \, \Omega_{MFNFM} \, \mu_{mic,1} \, \phi_{NH_4^+} \, \phi_{O_2} \, \phi_{pH} \, \phi_{ni} \]
The nitrifying microbial biomass saturates towards a maximum \( C_{max} \) (smooth limitation, continuous in value and slope at \( C_{mic,1} = C_{max}/2 \)):
\[C_{nit} = \begin{cases} C_{mic,1} & \text{if } C_{mic,1} < C_{max}/2 \\ C_{max} - \frac{C_{max}}{1 + \left( \frac{2 \, C_{mic,1}}{C_{max}} \right)^2} & \text{otherwise} \end{cases} , \qquad C_{max} = \Omega_{MFNMM} \cdot h \]
The consumed oxygen is taken proportionally from the gaseous and the dissolved \( O_2 \) pool.
The influence of \( NH_4^+ \) (aerobic soil volume) on nitrification of \( NH_4^+ \) is given by:
\[\phi_{NH_4^+} = \frac{NH_4^+}{NH_4^+ + \Omega_{MKNHN} \cdot V_{ae} \cdot h} \]
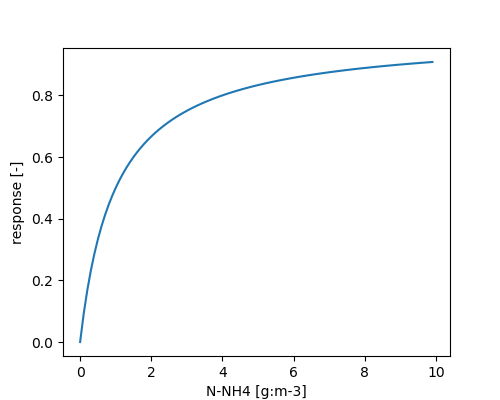
The influence of \( O_2 \) (gaseous and dissolved) on nitrification of \( NH_4^+ \) is given by:
\[\phi_{O_2} = \frac{O_2}{O_2 + \Omega_{MKON} \cdot h} \]
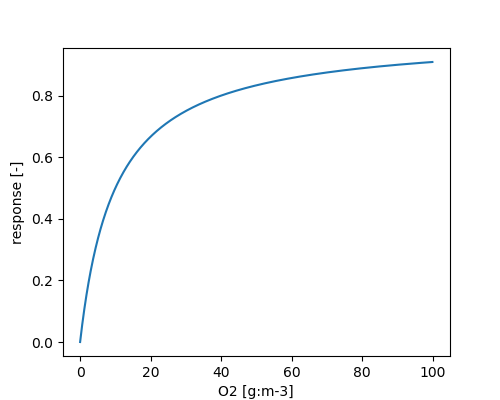
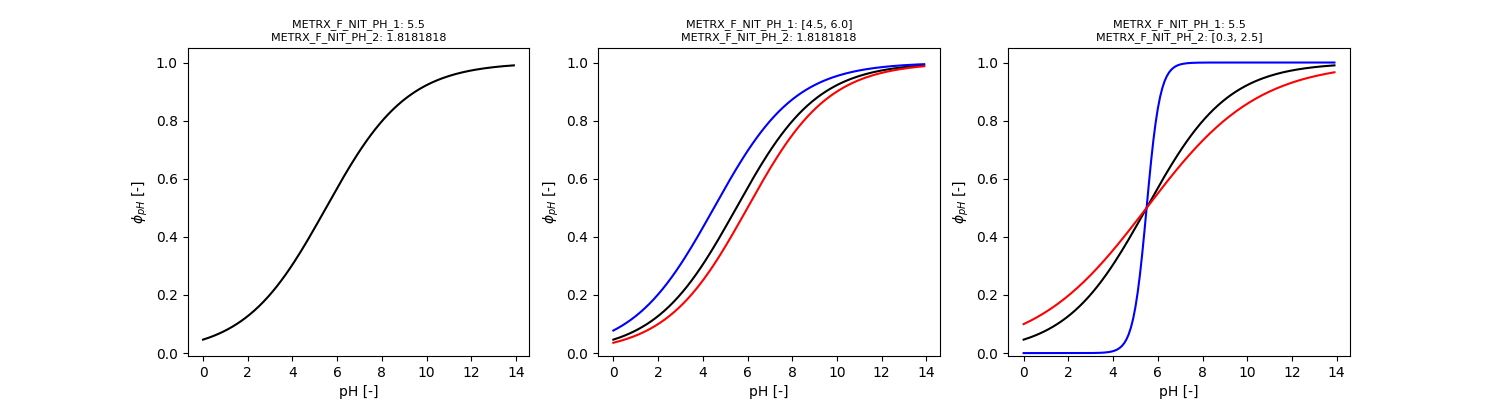
The influence of pH on nitrification of \( NH_4^+ \) is given by a logistic function, representing the inhibition of nitrifiers at low pH:
\[\phi_{pH} = \frac{1}{1 + e^{-\frac{pH - \Omega_{MFNP1}}{\Omega_{MFNP2}}}} \]
The influence of nitrification inhibitors \( \phi_{ni} = \max(0, 1 - I_{ni}) \) with the inhibition \( I_{ni} \) is given by Enhanced efficiency nitrogen fertilizers.
During the first step of nitrification a certain amount of N is lost in form of \( NO \) and \( N_2O \). The relevant processes are a mix of:
Reported production of \( NO \) during nitrification:
All \( N_2O \) produced in connection with nitrification was initially \( NO \). Emissions of \( NO \) and \( N_2O \) during nitrification are likely influenced by soil temperature and moisture (Chen et al. 2010):
\[N_{NO+N_2O} = \Omega_{MKNNN} \cdot \phi_{NO+N2O, T, wfps} \cdot N_{nit} \]
The remaining nitrified nitrogen \( N_{nit} - N_{NO+N_2O} \) is released as \( NO_2^- \). \( NO \) and \( N_2O \) are directly added to the gas phase of the soil layer. Soil water is expressed as water filled pore space ( \( wfps = \theta / \theta_{sat} \)).
The associated factor \( \phi_{NO+N2O, T, wfps} \) is given by a harmonic mean of a soil temperature ( \( \phi_{NO+N2O, T} \)) and a soil water ( \( \phi_{NO+N2O, wfps} \)) depending response coefficient:
\[\phi_{NO+N2O, T, wfps} = \frac{2.0}{\frac{1.0}{\phi_{NO+N2O, T}} + \frac{1.0}{\phi_{NO+N2O, wfps}}} \]
with \( \phi_{NO+N2O, T}\) given by:
\[\phi_{NO+N2O, T} = \frac{g_T}{\left(1 + g_T^4\right)^{1/4}}, \qquad g_T = \Omega_{MFNNNTE1} \cdot e^{\frac{T}{\Omega_{MFNNNTE2}}} \]
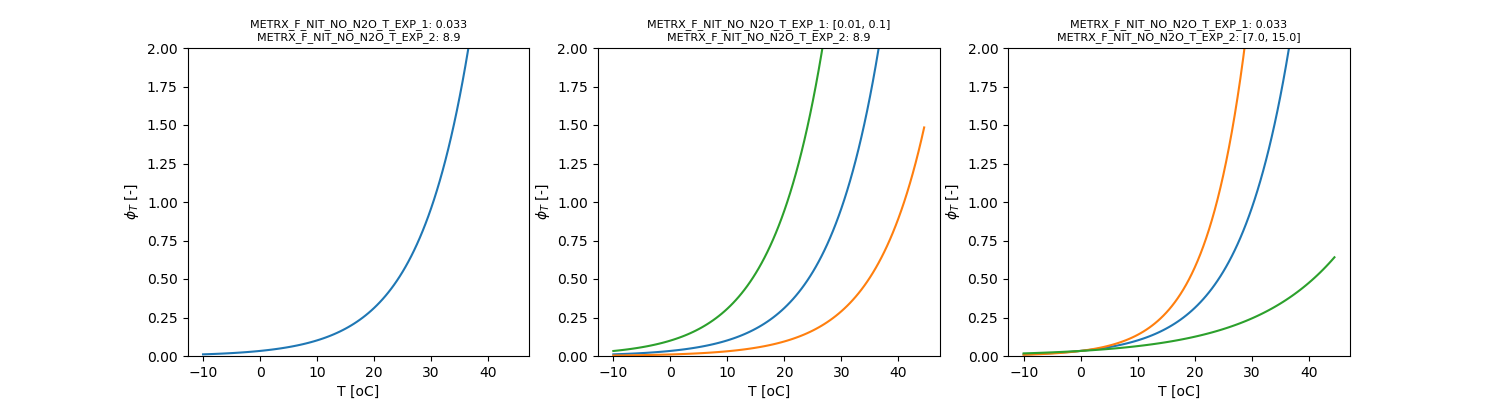
and with \( \phi_{NO+N2O, wfps}\) given by:
\[ \phi_{NO+N2O, wfps} = 1 - \frac{1}{1 + e^{(wfps - \Omega_{MFNNNMW1}) \cdot \Omega_{MFNNNMW2}}} \]
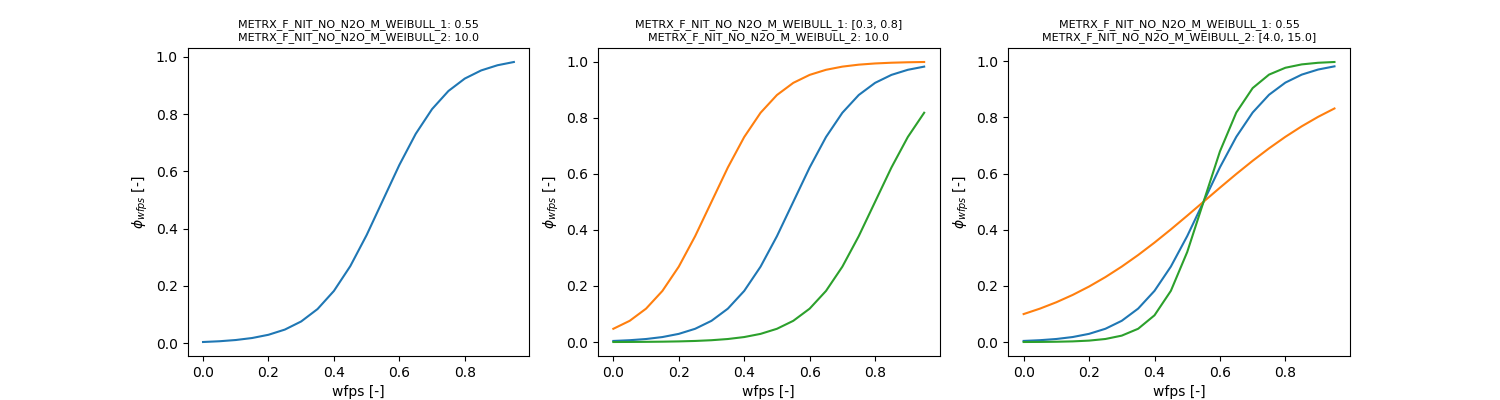
The fraction of \( NO \) decreases with increasing soil water, the remainder is released as \( N_2O \):
\begin{eqnarray*}N_{NO} &=& N_{NO+N_2O} \cdot \phi_{NO, wfps} \\ N_{N_2O} &=& N_{NO+N_2O} \cdot (1 - \phi_{NO, wfps}) \end{eqnarray*}
with
\[\phi_{NO, wfps} = 1 - \frac{1}{ 1 + e^{-\Omega_{MFNNME1} \cdot (wfps - \Omega_{MFNNME2})}} \]
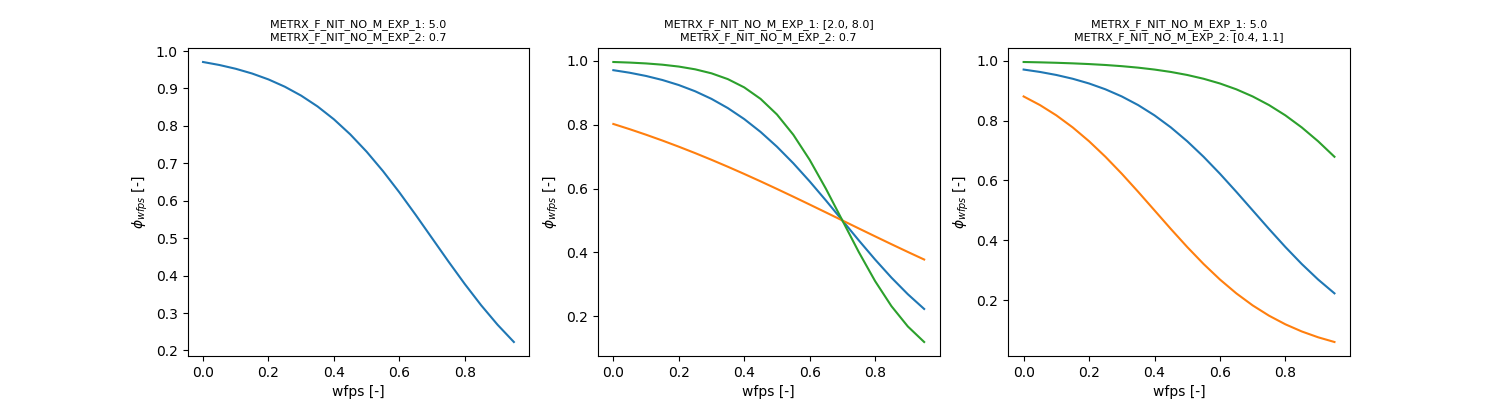
No pH effect of ammonia oxidation on N2O emissions observed (Booth, Stark and Rastetter 2005).
The second step of nitrification (oxidation of \( NO_2^- \) to \( NO_3^- \) in the aerobic soil volume) is calculated independent of microbial biomass. In each time step, the following amount of \( NO_2^- \) is oxidised:
\[N_{NO_2^- \rightarrow NO_3^-} = 0.9 \, NO_2^- \cdot \frac{NO_2^-}{NO_2^- + \Omega_{MKNON} \cdot V_{ae} \cdot h} \]
This represents the generally fast turnover of \( NO_2^- \) in soils, which prevents its accumulation.
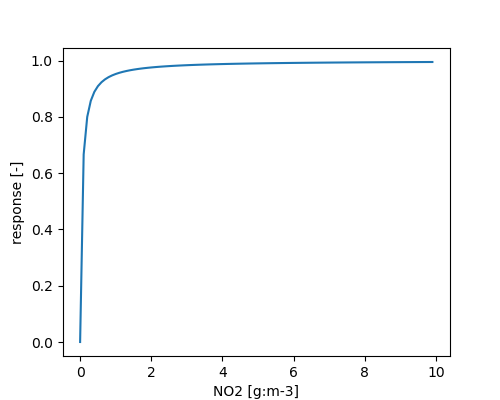
Denitrification is calculated as a four-step reduction of nitrogen oxides by heterotrophic, facultatively anaerobic microbes (denitrifier biomass \( C_{mic,2} \)):
\[NO_3^- \rightarrow NO_2^- \rightarrow NO \rightarrow N_2O \rightarrow N_2 \]
Denitrifiers live in the anaerobic soil volume fraction \( V_{an} \), i.e., all substrates (DOC, acetate, \( NO_3^-, NO_2^-, NO, N_2O \)) refer to the respective pools of the anaerobic soil volume. For each soil layer and time step the following sequence is calculated:
All denitrification steps are calculated based on the actively denitrifying microbial biomass \( C_{mic,2} \cdot a_{mic} \). The activity coefficient of denitrifying microbes \( a_{mic} \) depends on soil temperature and soil moisture.
The temperature and moisture dependency of denitrifying microbes is given by the harmonic mean of a soil temperature ( \( \phi_{T}\)) and a soil moisture ( \( \phi_{\theta}\)) response coefficient.
\[a_{mic} = \frac{2}{\frac{1}{\phi_{T}} + \frac{1}{\phi_{\theta}}} \]
The soil temperature response \( \phi_{T}\) of denitrification is given by the same temperature dependency as for general microbial activity:
\[\phi_{T} = e^{-\Omega_{MFMTE1} \cdot \left( 1 - \frac{T}{\Omega_{MFMTE2}} \right)^2} \]
If the option freezethaw is set to ft_processes, \( \Omega_{MFMTE1} \) is replaced by a temperature dependent coefficient that shifts between \( \Omega_{MFMTEC} \) and \( \Omega_{MFMTE1} \):
\[\Omega_{MFMTEC} + \frac{\Omega_{MFMTE1} - \Omega_{MFMTEC}}{1 + e^{-\Omega_{MFMTE1} (T - \Omega_{MFMTE2})}} \]
The soil moisture response \( \phi_{\theta}\) of denitrification is given by a logistic function of the water content relative to field capacity ( \( \theta_{rel} = \theta / \theta_{fc} \)):
\[ \phi_{\theta} = 1 - \frac{1}{1 + e^{(\theta_{rel} - \Omega_{MFDMW1}) \cdot \Omega_{MFDMW2}}} \]
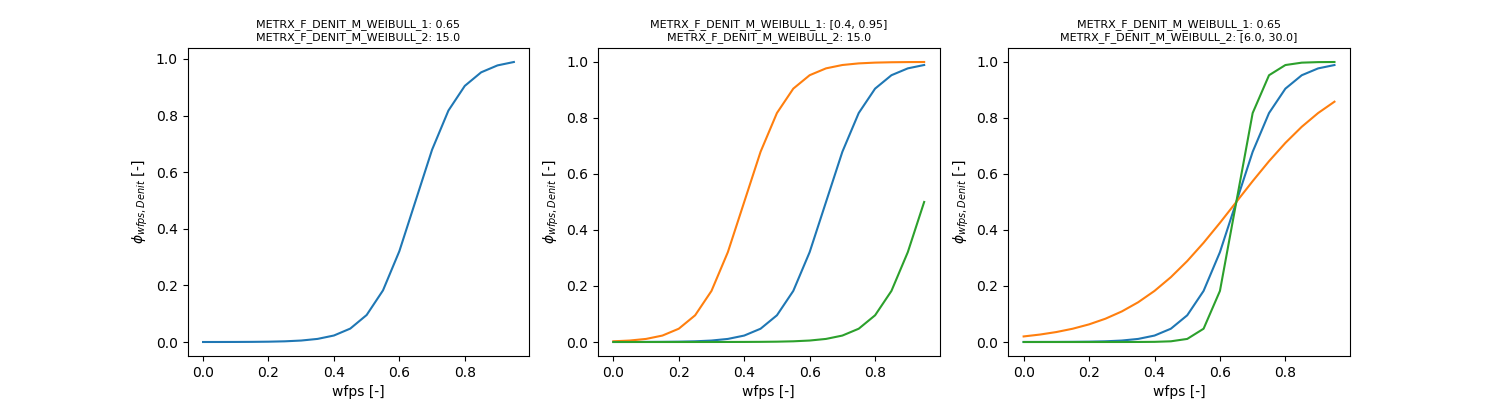
Denitrifier growth depends on the availability of carbon (DOC and acetate) and of oxidised nitrogen serving as electron acceptor ( \( N_{ox} \)):
\begin{eqnarray*}N_{ox} &=& NO_3^- + NO_2^- + NO + N_2O \\ \phi_{C} &=& \frac{DOC + Ac}{DOC + Ac + K_{C}} \\ \phi_{N} &=& \frac{N_{ox}}{N_{ox} + K_{N}} \\ \phi_{C,N} &=& \frac{2}{\frac{1}{\phi_{C}} + \frac{1}{\phi_{N}}} \end{eqnarray*}
The Michaelis-Menten constants are given as concentrations and are converted into amounts within the anaerobic volume of the soil layer (layer thickness \( h \)):
\begin{eqnarray*}K_{C} &=& \Omega_{MKCD} \cdot V_{an} \cdot h \\ K_{N} &=& \Omega_{MKND} \cdot V_{an} \cdot h \end{eqnarray*}
Microbial enzymes relevant for denitrification are:
Heterotrophic denitrification decreases with decreasing pH. Low pH inhibits all enzymes but especially nosZ. The general pH influence on denitrifier growth (affecting all enzymes) is given by a logistic function increasing with pH:
\[\phi_{pH} = 1 - \frac{1}{1 + e^{\frac{pH - \Omega_{MFDP1}}{\Omega_{MFDP2}}}} \]
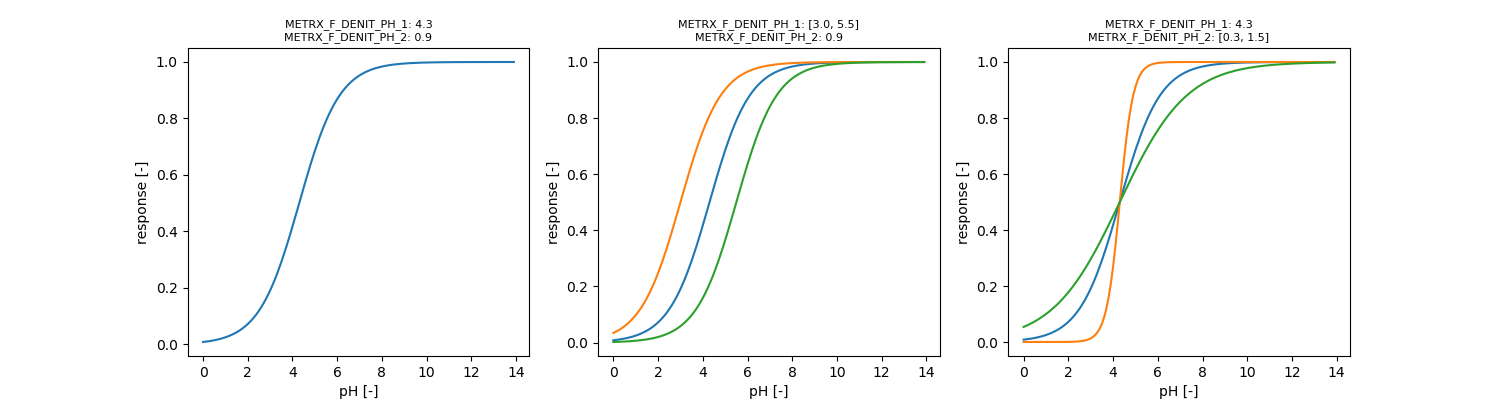
The additional pH dependency of nosZ, i.e., of the reduction of \( N_2O \) to \( N_2 \), is given by:
\[\phi_{pH,nosZ} = 1 - \frac{1}{1 + e^{\frac{pH - \Omega_{MFDNP1}}{\Omega_{MFDNP2}}}} \]
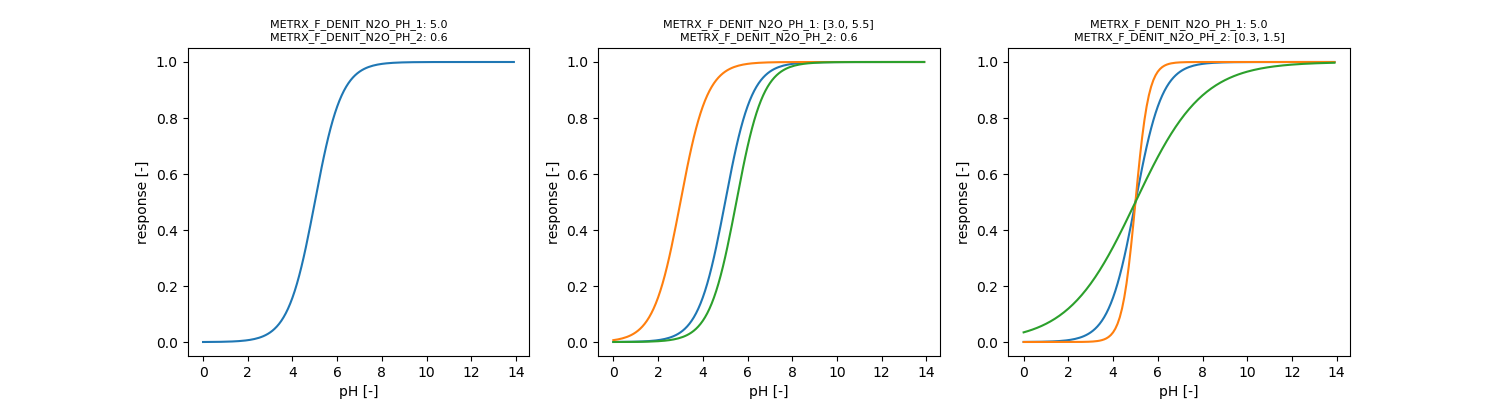
If the option freezethaw is set to yes, \( N_2O \) reduction is additionally inhibited at low soil temperatures:
\[\phi_{T,nosZ} = \frac{1}{1 + e^{-\frac{T - 10}{2}}} \]
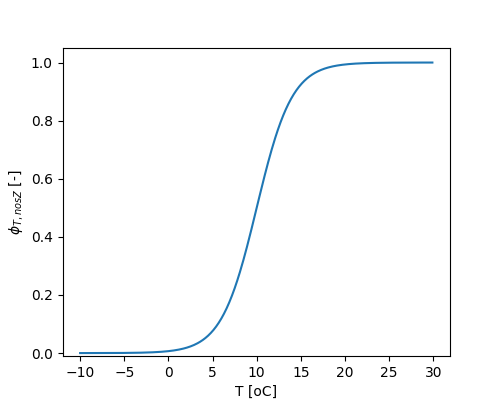
Both factors are combined to \( \phi_{nosZ} = \phi_{pH,nosZ} \cdot \phi_{T,nosZ} \).
Total microbial carbon demand includes assimilation and dissimilation:
\begin{eqnarray*}C_{demand} &=& C_{mic,2} \, \mu_{mic,2} \, a_{mic} \frac{1}{Y_{denit}} \phi_{C,N} \phi_{pH} \\ C_{assi} &=& C_{demand} \, Y_{denit} \\ C_{diss} &=& C_{demand} \, (1 - Y_{denit}) \end{eqnarray*}
The dissimilated carbon \( C_{diss} \) is allocated to the electron acceptors \( NO_3^-, NO_2^-, NO \) and \( N_2O \) with the fractions \( \psi_i \left ( \sum \psi_i = 1 \right ) \). The use of \( NO_3^- \) is suppressed by the availability of the intermediates \( N_{int} \), and \( N_2O \) is only available as electron acceptor as far as nosZ is not inhibited:
\begin{eqnarray*}N_{int} &=& NO_2^- + NO + \phi_{nosZ} \, N_2O \\ \psi_{NO_3^-} &=& \left( 1 - \frac{N_{int}}{N_{int} + K_{N}} \right) \frac{NO_3^-}{N_{ox}} \\ \psi_{NO_2^-} &=& (1- \psi_{NO_3^-}) \cdot \frac{NO_2^-}{N_{int}} \\ \psi_{NO} &=& (1- \psi_{NO_3^-}) \cdot \frac{NO}{N_{int}} \\ \psi_{N_2O} &=& (1- \psi_{NO_3^-}) \cdot \frac{\phi_{nosZ} \, N_2O}{N_{int}} \end{eqnarray*}
The suppression of \( NO_3^- \) use by the intermediates accounts for the spatial heterogeneity of denitrification in soils, which is not resolved by the model. \( NO_3^- \) in the soil is assumed to be homogeneously distributed. Once microbes with access to \( NO_3^- \) start denitrifying under low \( O_2 \) availability, the produced intermediates ( \( NO_2^-, NO, N_2O \)) are in close vicinity of the denitrifying microbes, i.e., their local concentration at the active sites is higher than the average concentration of the soil layer. Hence, with the build up of intermediates, \( NO_3^- \) is weighted less as electron acceptor.
An alternative formulation (currently commented in the code) uses a constant local enrichment factor \( \omega \) of the intermediates relative to \( NO_3^- \), which is independent of the absolute amount of nitrogen:
\[\psi_{NO_3^-} = \frac{NO_3^-}{NO_3^- + \omega \, N_{int}} \]
\( NO_2^- \) and \( NO \) can be reduced by a single step or by multiple steps before the product is released from the denitrifying organism to the soil environment. The fraction that is completely reduced to \( N_2 \) within the same organism increases linearly with the anaerobic volume fraction (assuming that denitrification enzymes are more developed under anaerobic conditions):
\[\phi_{anvf,1} = \Omega_{MFDN1} \cdot \Omega_{MFDN2} + V_{an} \cdot (\Omega_{MFDN2} - \Omega_{MFDN1} \cdot \Omega_{MFDN2}) \]
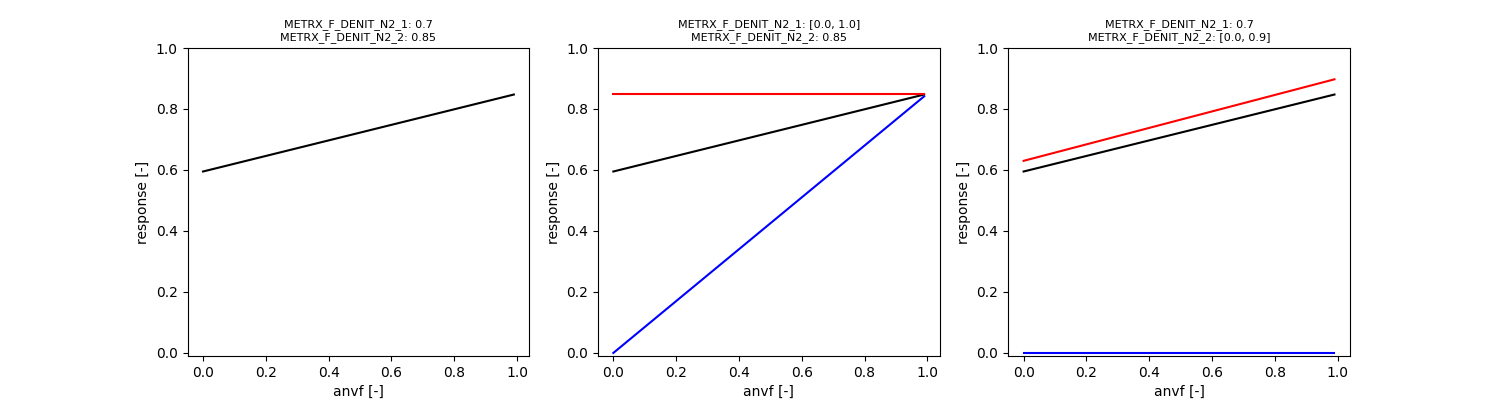
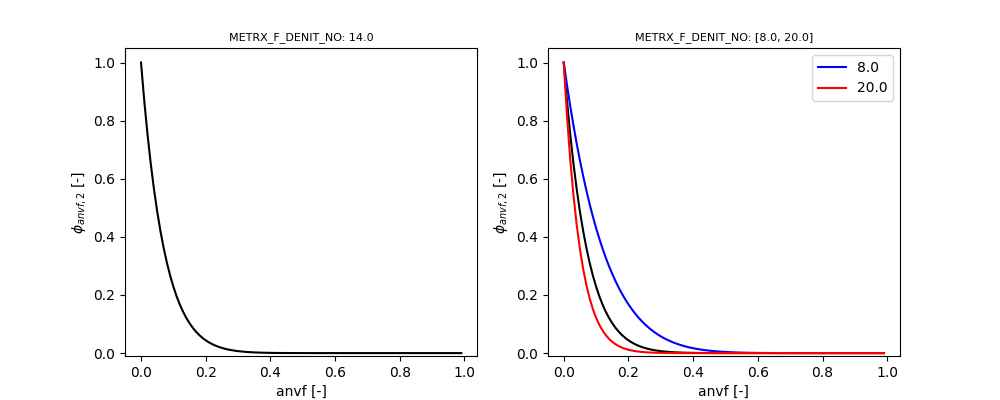
Of the remaining fraction, the share released as \( NO \) after reduction of \( NO_2^- \) decreases strongly with increasing anaerobic volume fraction:
\[\phi_{anvf,2} = (1 - V_{an})^{\Omega_{MFDNO}} \]
The stoichiometry between reduced nitrogen and dissimilated carbon follows from the electron balance. The electrons of the consumed substrate carbon are either stored in the new biomass or transferred to the nitrogen oxides. Using the degree of reduction \( \gamma \) (mol electrons released per mol C upon complete oxidation to \( CO_2 \)), the electrons transferred to nitrogen oxides per mol of dissimilated carbon are:
\[e_{diss} = \frac{\gamma_{DOC} - Y_{denit} \, \gamma_{mic}}{1 - Y_{denit}} \]
With \( n_e \) electrons accepted per N atom of a reaction, the mass ratio of reduced nitrogen to dissimilated carbon is:
\[\xi_{CN} = \frac{e_{diss}}{n_e} \frac{M_N}{M_C} \]
| reaction | \( n_e \) |
|---|---|
| \( NO_3^- \rightarrow NO_2^- \) | 2 |
| \( NO_2^- \rightarrow NO \) | 1 |
| \( NO_2^- \rightarrow N_2O \) | 2 |
| \( NO_2^- \rightarrow N_2 \) | 3 |
| \( NO \rightarrow N_2O \) | 1 |
| \( NO \rightarrow N_2 \) | 2 |
| \( N_2O \rightarrow N_2 \) | 1 |
\begin{eqnarray*}C_{NO_3^-} &=& \psi_{NO_3^-} \cdot C_{diss} \\ N_{NO_3^- \rightarrow NO_2^-} &=& \xi_{CN, NO_3^- \rightarrow NO_2^-} \cdot C_{NO_3^-} \end{eqnarray*}
Reduced \( NO_2^- \) is released as \( NO, N_2O \) or \( N_2 \) depending on the anaerobicity of the soil and on the inhibition of nosZ. The associated carbon is given by:
\begin{eqnarray*}C_{NO_2^-} &=& \psi_{NO_2^-} \cdot C_{diss} \\ C_{NO_2^- \rightarrow N_2} &=& C_{NO_2^-} \cdot \phi_{anvf,1} \cdot \phi_{nosZ} \\ C_{NO_2^- \rightarrow NO} &=& C_{NO_2^-} \cdot (1-\phi_{anvf,1}) \cdot \phi_{anvf,2} \\ C_{NO_2^- \rightarrow N_2O} &=& C_{NO_2^-} - C_{NO_2^- \rightarrow N_2} - C_{NO_2^- \rightarrow NO} \end{eqnarray*}
The reduced nitrogen is given by:
\begin{eqnarray*}N_{NO_2^- \rightarrow N_2} &=& \xi_{CN, NO_2^- \rightarrow N_2} \cdot C_{NO_2^- \rightarrow N_2} \\ N_{NO_2^- \rightarrow NO} &=& \xi_{CN, NO_2^- \rightarrow NO} \cdot C_{NO_2^- \rightarrow NO} \\ N_{NO_2^- \rightarrow N_2O} &=& \xi_{CN, NO_2^- \rightarrow N_2O} \cdot C_{NO_2^- \rightarrow N_2O} \end{eqnarray*}
Reduced \( NO \) is released as \( N_2O \) or \( N_2 \) depending on the anaerobicity of the soil and on the inhibition of nosZ. The associated carbon is given by:
\begin{eqnarray*}C_{NO} &=& \psi_{NO} \cdot C_{diss} \\ C_{NO \rightarrow N_2} &=& C_{NO} \cdot \phi_{anvf,1} \cdot \phi_{nosZ} \\ C_{NO \rightarrow N_2O} &=& C_{NO} - C_{NO \rightarrow N_2} \end{eqnarray*}
The reduced nitrogen is given by:
\begin{eqnarray*}N_{NO \rightarrow N_2} &=& \xi_{CN, NO \rightarrow N_2} \cdot C_{NO \rightarrow N_2} \\ N_{NO \rightarrow N_2O} &=& \xi_{CN, NO \rightarrow N_2O} \cdot C_{NO \rightarrow N_2O} \end{eqnarray*}
\( N_2O \) taken up from the soil is completely reduced to \( N_2 \) (the inhibition of nosZ is already considered in \( \psi_{N_2O} \)):
\begin{eqnarray*}C_{N_2O} &=& \psi_{N_2O} \cdot C_{diss} \\ N_{N_2O \rightarrow N_2} &=& \xi_{CN, N_2O \rightarrow N_2} \cdot C_{N_2O} \end{eqnarray*}
Denitrifiers assimilate \( NH_4^+ \), \( NO_3^- \) and DON of the anaerobic soil volume towards their optimum C:N ratio, limited by their activity \( a_{mic} \) and by nitrogen availability (Michaelis-Menten constant METRX_KMM_N_MIC, scaled to the anaerobic volume as above).
Death of denitrifiers decreases with carbon availability:
\[C_{death} = \frac{C_{mic,2} \, a_{mic} \, A_{max,2}}{1 + (DOC + Ac) \frac{\Omega_{MKAC}}{V_{an} \, h}} \]
Nitrogen of dead biomass follows the current microbial C:N ratio. The fraction METRX_FRAC_MINERAL is directly mineralized to \( NH_4^+ \), the remainder is allocated to dead organic matter.
At low pH, \( NO \) and \( N_2O \) can be produced via chemical decomposition of hydroxylamine ( \( NH_2OH \)), nitroxyl hydride (HNO) or \( NO_2^- \), which are intermediate products of ammonia oxidation (Zumft 1997; Wrage et al. 2001). In MeTrX, only the chemical decomposition of \( NO_2^- \) to \( NO \) is considered. It is calculated in both the aerobic and the anaerobic soil volume:
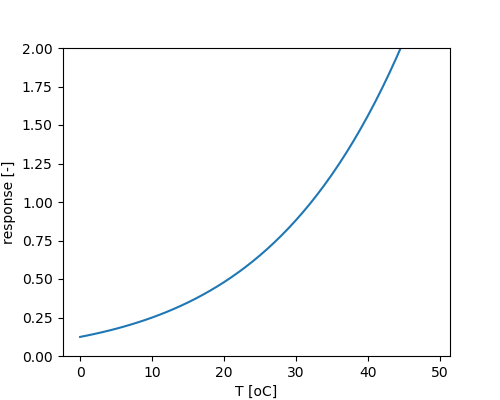
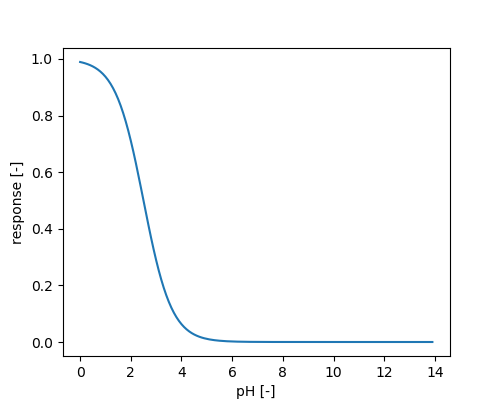
\begin{eqnarray*} \frac{d NO_2^-}{dt} &=& - K_{MKDC} \cdot \phi_{T} \cdot \phi_{pH} \cdot NO_2^- \\ \phi_{T} &=& \Omega_{MFCT1} \cdot e^{-\frac{\Omega_{MFCT2}}{R \, (T + 273.15)}} \\ \phi_{pH} &=& \frac{1}{1 + e^{\frac{pH - \Omega_{MFCP1}}{\Omega_{MFCP2}}}} \end{eqnarray*}
Temperature dependency of chemodenitrification:
pH dependency of chemodenitrification:
Under anaerobic conditions acetate and hydrogen are produced, which may serve as substrate for iron reducing and methanogenic bacteria.
Temperature dependency of microbial activity:
The stoecheometry of iron reduction via aceate is given by::
\[ CHCOO^- + 8 Fe^{3+} + 4 H_2O \rightarrow 2 HCO_3^- + 8 Fe^{2+} + 9 H^+ \]
The stoecheometry of iron reduction via aceate is given by::
\[ H_2 + 2 Fe^{3+} + 4 H^+ \rightarrow 2 Fe^{2+} + 6 H_2O \]
Iron reduction via acetate and hydrogen depends on the amount of Fe3+ and the amount of either aceatet or hydrogen each modeled using a Michaelis Menten kinetic. Further influencing factors are temperature, NO3 and O2:
\[ \frac{dFe^{3+}}{dt} = - METRX\_MUEMAX\_C\_FE\_RED \cdot \phi_{T} \cdot \phi_{NO3} \cdot \phi_{O2} \cdot \phi_{Fe3+} \cdot \phi_{AC/H2} \]
The dependy on NO3 is given by:
\[ \phi_{NO3} = 1 - \frac{NO3}{NO3 + NO3\_MOLAR\_MAX\_FE\_RED} \]
The stoecheometry of iron oxidation is given by::
\[ 4 Fe^{2+} + O_2 + 10 H_2O \rightarrow 4 Fe(OH)_3 + 8 H^+ \]
\[ \frac{dFe^{2+}}{dt} = - METRX\_KR\_OX\_FE \cdot Fe^{2+} \cdot \phi_{O2} \]
The dependy on O2 is given by:
\[ \phi_{O2} = \frac{O_2}{O_2 + METRX\_KMM\_O2\_FE\_OX} \]
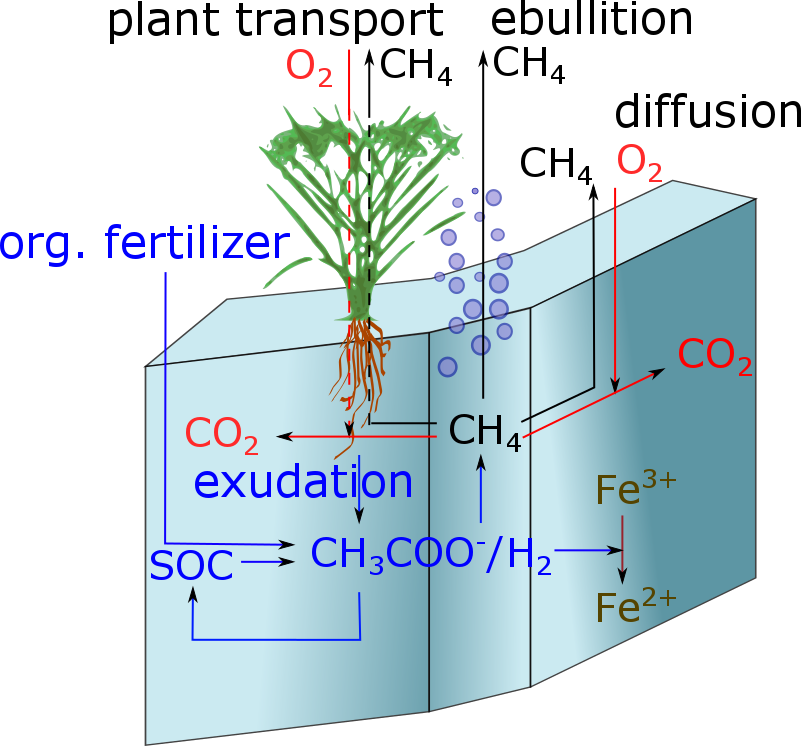
Methane is produced by methanogenic archaea in the anaerobic soil volume \( V_{an} \) via two pathways:
Both substrates are produced by fermentation (see Fermentation and synthrophy). Methanogenic biomass is not simulated explicitly. Produced methane is added to the dissolved methane pool of the soil layer.
Methanogens are outcompeted by iron reducers. Therefore, methane is only produced after a large fraction of total iron has been reduced (see Iron reduction):
\[ Fe^{3+} \le \Omega_{MFFCP} \cdot (Fe^{3+} + Fe^{2+}) \]
Both pathways depend on soil temperature, soil moisture, pH, nitrate and soil depth.
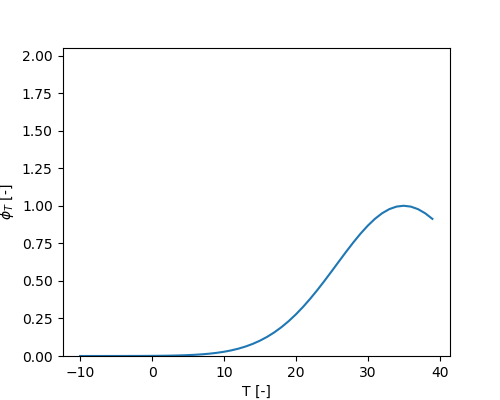
Temperature
\[ \phi_{T} = e^{-\Omega_{MFCPTE1} \left( 1 - \frac{T}{\Omega_{MFCPTE2}} \right)^2} \]
Moisture
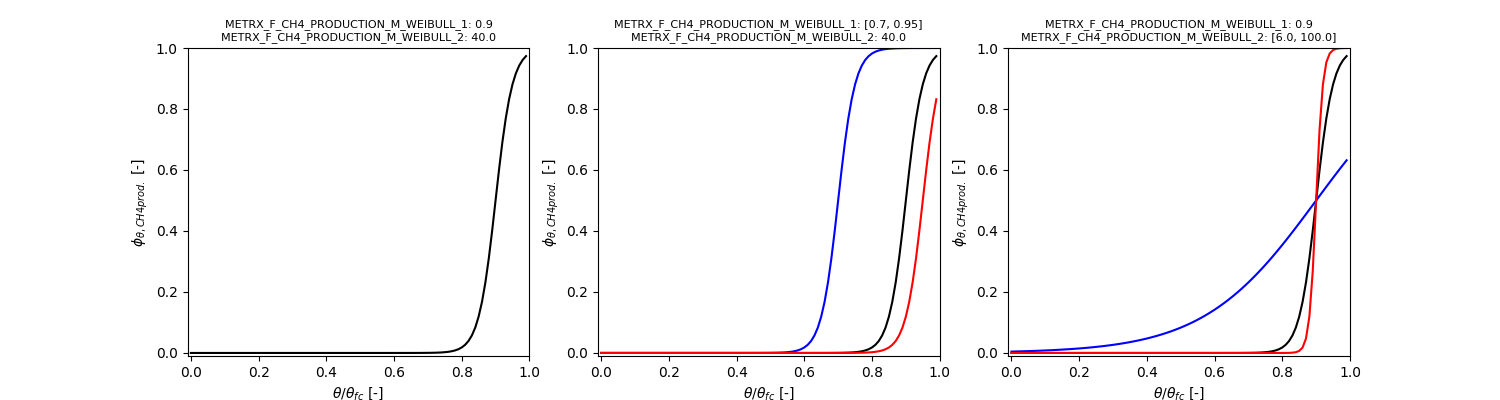
The moisture response is given by a logistic function of the water content relative to field capacity ( \( \theta_{rel} = \theta / \theta_{fc} \), bounded to [0.001, 0.999]):
\[ \phi_{\theta} = 1 - \frac{1}{1 + e^{(\theta_{rel} - \Omega_{MFCPMW1}) \cdot \Omega_{MFCPMW2}}} \]
pH value
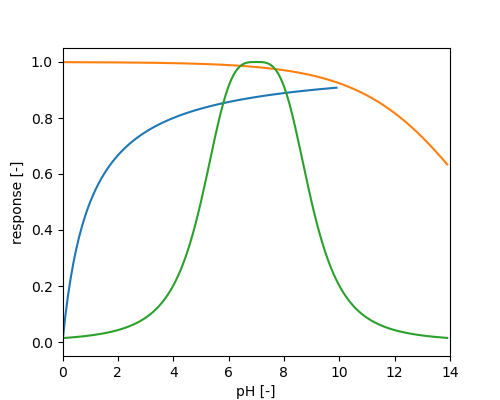
\[ \phi_{pH} = \frac{1}{1 + \left( \frac{|pH - \Omega_{MFCP3}|}{\Omega_{MFCP1}} \right)^{\Omega_{MFCP2}}} \]
Nitrate
Methane production is inhibited by nitrate in the anaerobic soil volume ( \( NO_3^- \) [kgN m-2]) in the same way as iron reduction:
\[ \phi_{NO_3} = 1 - \frac{NO_3^-}{NO_3^- + K_{NO_3}}, \qquad K_{NO_3} = 10^{-4} \, \mathrm{mol \, m^{-3}} \cdot h \]
with layer thickness \( h \) [m].
Depth
Since methanogenic biomass is not simulated explicitly, its decrease with soil depth \( z \) [m] (lower boundary of the soil layer) is given by:
\[ \phi_{z} = \frac{1}{1 + e^{10 \, (z - 0.4)}} \]
i.e., methane production is reduced by 50% at 0.4 m depth and by more than 99% below 0.86 m.

All factors are combined multiplicatively:
\[ \phi_{env} = \phi_{T} \cdot \phi_{\theta} \cdot \phi_{pH} \cdot \phi_{NO_3} \cdot \phi_{z} \]
Acetate is split into methane and carbon dioxide, i.e., half of the acetate carbon is released as \( CH_4 \):
\[ CH_3COOH \rightarrow CO_2 + CH_4 \]
\[ \frac{d CH_{4,Ac}}{d t} = \Omega_{MMCCP} \cdot h \cdot \phi_{Ac} \cdot \phi_{env} \]
with acetate \( Ac \) [kgC m-2] in the anaerobic soil volume. The upper limit ensures that at most 90% of the available acetate carbon is consumed per time step ( \( CH_4 \) and \( CO_2 \) carbon). The dependency on acetate \( \phi_{Ac} \) is given by a Michaelis-Menten kinetic with the half saturation constant given as concentration within the anaerobic soil volume:
\[ \phi_{Ac} = \frac{Ac}{\Omega_{MKACP} \cdot V_{an} \cdot h + Ac} \]
Hydrogen is used to reduce dissolved carbon dioxide:
\[ 4 H_2 + CO_2 \rightarrow 2 H_2O + CH_4 \]
\[ \frac{d CH_{4,H_2}}{d t} = \Omega_{MMHCP} \cdot h \cdot \phi_{H_2} \cdot \phi_{env}, \; 0.9 \cdot c_{H_2} \cdot H_2 \]
with \( c_{H_2} = M_C / (4 \, M_{H_2}) \) converting hydrogen [kg m-2] into methane carbon [kgC m-2] and the upper limit ensuring that at most 90% of the limiting substrate ( \( H_2 \) or dissolved \( CO_2 \)) is consumed per time step. The dependency on hydrogen \( \phi_{H_2} \) is given by a Michaelis-Menten kinetic with the half saturation constant given as concentration within the anaerobic soil volume (as for acetate, fermentation and iron reduction):
\[ \phi_{H_2} = \frac{H_2}{\Omega_{MKHCP} \cdot V_{an} \cdot h + H_2} \]
Methane is oxidised by aerobic methanotrophic bacteria. The stoichiometry of methanotrophy is given by:
\[ CH_4 + (2-\alpha) O_2 \rightarrow (1-\alpha) CO_2 + (2-\alpha) H_2O + \alpha CH_2O \]
i.e., the fraction \( \alpha \) of oxidised methane carbon is assimilated into microbial biomass ( \( C_{mic,1} \)), the remainder is released as \( CO_2 \), and \( 2-\alpha \) mol \( O_2 \) are consumed per mol \( CH_4 \).
Methane oxidation is calculated for total methane ( \( CH_4 \), gaseous and dissolved) and total oxygen ( \( O_2 \), gaseous and dissolved) of a soil layer. Consumption of \( CH_4 \) and \( O_2 \) is distributed proportionally to the gaseous and dissolved pools.
Methane oxidation depends on soil temperature, soil moisture, pH, oxygen, methane and nitrogen.
Temperature
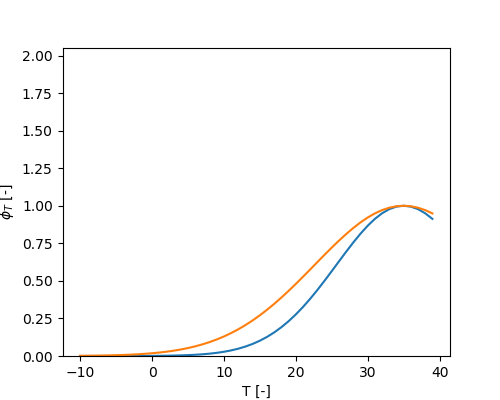
\[ \phi_{T} = e^{-\Omega_{MFCOTE1} \left( 1 - \frac{T}{\Omega_{MFCOTE2}} \right)^2} \]
Moisture
The moisture response \( \phi_{\theta} \) is the same as for general microbial activity (see Temperature and moisture dependency of microbial growth), i.e., a logistic function of the water content relative to field capacity with parameters METRX_F_MIC_M_WEIBULL_1 and METRX_F_MIC_M_WEIBULL_2.
pH value
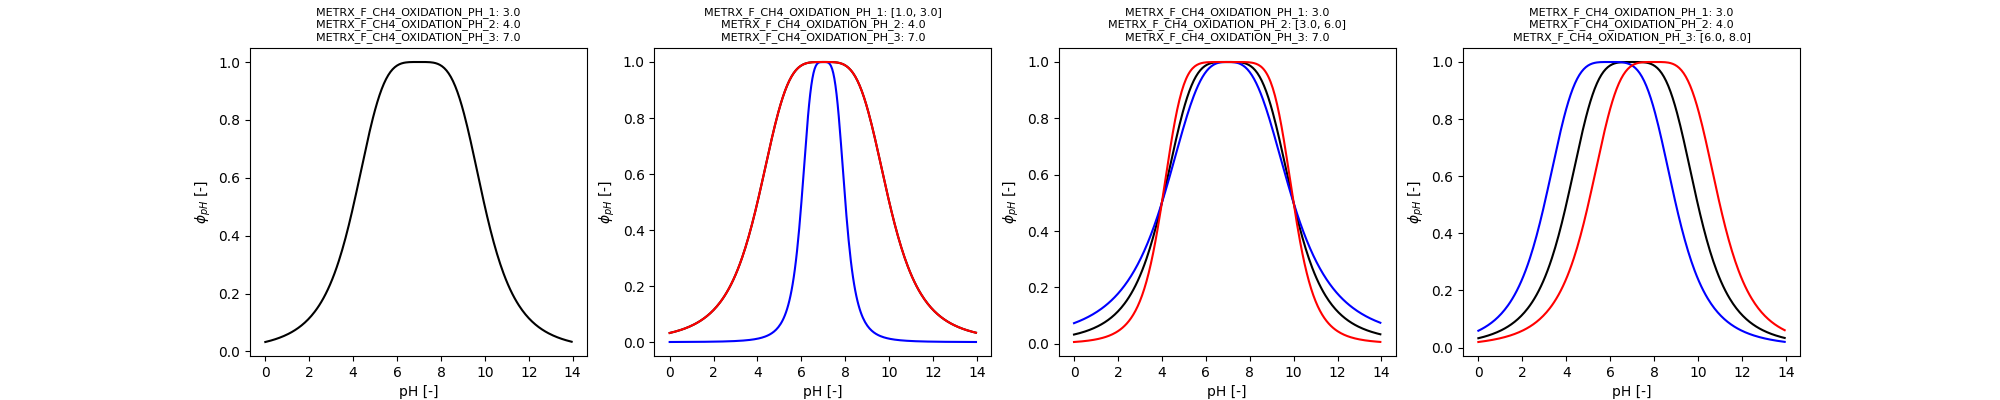
\[ \phi_{pH} = \frac{1}{1 + \left( \frac{|pH - \Omega_{MFCO3}|}{\Omega_{MFCO1}} \right)^{\Omega_{MFCO2}}} \]
Oxygen, methane and nitrogen
Substrate dependencies are given by Michaelis-Menten kinetics with half saturation constants given as concentrations and converted into amounts of the soil layer (layer thickness \( h \)):
\begin{eqnarray*} \phi_{O_2} &=& \frac{O_2}{\Omega_{MKOCO} \cdot h + O_2} \\ \phi_{CH_4,HA} &=& \frac{CH_4}{\Omega_{MKCCOHA} \cdot h + CH_4} \\ \phi_{CH_4,LA} &=& \frac{CH_4}{\Omega_{MKCCOLA} \cdot h + CH_4} \\ \phi_{N} &=& (1- \Omega_{MFNCO}) + \Omega_{MFNCO} \frac{N}{\Omega_{MKNCO} \cdot h + N} \end{eqnarray*}
with \( N = NH_4^+ + DON + NO_3^- \) (aerobic and anaerobic soil volume).
Two groups of methanotrophs are distinguished: low affinity methanotrophs (LA) being active at high methane concentrations (e.g., close to methanogenic zones) and high affinity methanotrophs (HA) oxidising methane at (sub-)atmospheric concentrations. Only low affinity methanotrophs depend on nitrogen availability:
\begin{eqnarray*} \frac{d CH_{4,LA}}{d t} &=& - \min \left( \Omega_{MMCCOLA} \cdot h \cdot \phi_{CH_4,LA} \cdot \phi_{T} \cdot \phi_{\theta} \cdot \phi_{pH} \cdot \phi_{O_2} \cdot \phi_{N}, \; CH_{4,max} \right) \\ \frac{d CH_{4,HA}}{d t} &=& - \min \left( \Omega_{MMCCOHA} \cdot h \cdot \phi_{CH_4,HA} \cdot \phi_{T} \cdot \phi_{\theta} \cdot \phi_{pH} \cdot \phi_{O_2}, \; CH_{4,max} \right) \\ CH_{4,max} &=& \min \left( CH_4, \; \frac{O_2}{c_{O_2}} \right) \end{eqnarray*}
The larger of both rates is applied. \( CH_{4,max} \) limits oxidation by the available methane and oxygen with \( c_{O_2} = (2 - \alpha) \, M_{O_2} / M_C \) [kgO2 kgC-1].
Algae growth is only considered if option "algae" is set true.
Algae growth only takes place if ponding water table exists and incoming shortwave radiation directly above soil (below canopy) is greater zero.
Algae growth rate depends on:
\[ \phi_N = (1.0 - \Phi_{METRX\_F\_N\_ALGAE}) + \Phi_{METRX\_F\_N\_ALGAE} \cdot \frac{N}{\Phi_{METRX\_KMM\_N\_ALGAE} + N } \]
\[ \phi_T = \left\{ \begin{array}{cccc} 0.0 & T \le 15.0 \\ \frac{T - 15.0}{15.0} & 15.0 < T \le 30.0 \\ 1.0 - \frac{T - 30.0}{15.0} & 30.0 < T \le 45.0 \\ 0.0 & 45.0 > T \end{array} \right. \label{eq2} \]
\[ \phi_P = 1.0 - e^{\frac{-P}{100.0}} \]
Algae growth rate is given by:
\[ \mu_g = \Phi_{METRX\_MUEMAX\_C\_ALGAE} \cdot min(\phi_N, \phi_T, \phi_P) \]
Algae growth changes pH value of the ponding water table:
\[ \Delta pH = 3.0 \cdot \phi_N \cdot \phi_T \cdot \phi_P \]
Algae turnover:
\[ \mu_d = m_A \cdot \Phi_{METRX\_AMAX\_ALGAE} \]
The chemical equilibrium between dissolved \( NH_3 \) and \( NH_4 \) is given by (Sadeghi et al., 1988):
\begin{eqnarray*}f_{NH_3} &=& \frac{c_{NH_3}}{c_{NH_3} + c_{NH_4}} \\ f_{NH_3} &=& \frac{1}{1 + \frac{10^{-pH}}{K_a}} \\ K_a &=& 10^{\frac{-2728.3}{T} - 0.094219} \end{eqnarray*}
The chemical equilibrium between dissolved \( NH_3 \) and \( NH_4 \) is calculated for the surface water table and the soil solution.
Ammonium is partly adsorped at the soil surface depending on soil texture.
The effective diffusion coefficient \( D_{eff} \) relates to the tortuosity of the soil matrix. Two different approaches can be chosen (see also Model options):
\[ D_{eff} = \theta_{g}^{\Omega_{MDEEA}} \]
\[ D_{eff} = \frac{\theta_{g}^{10/3}}{\theta_{p}^2} \]
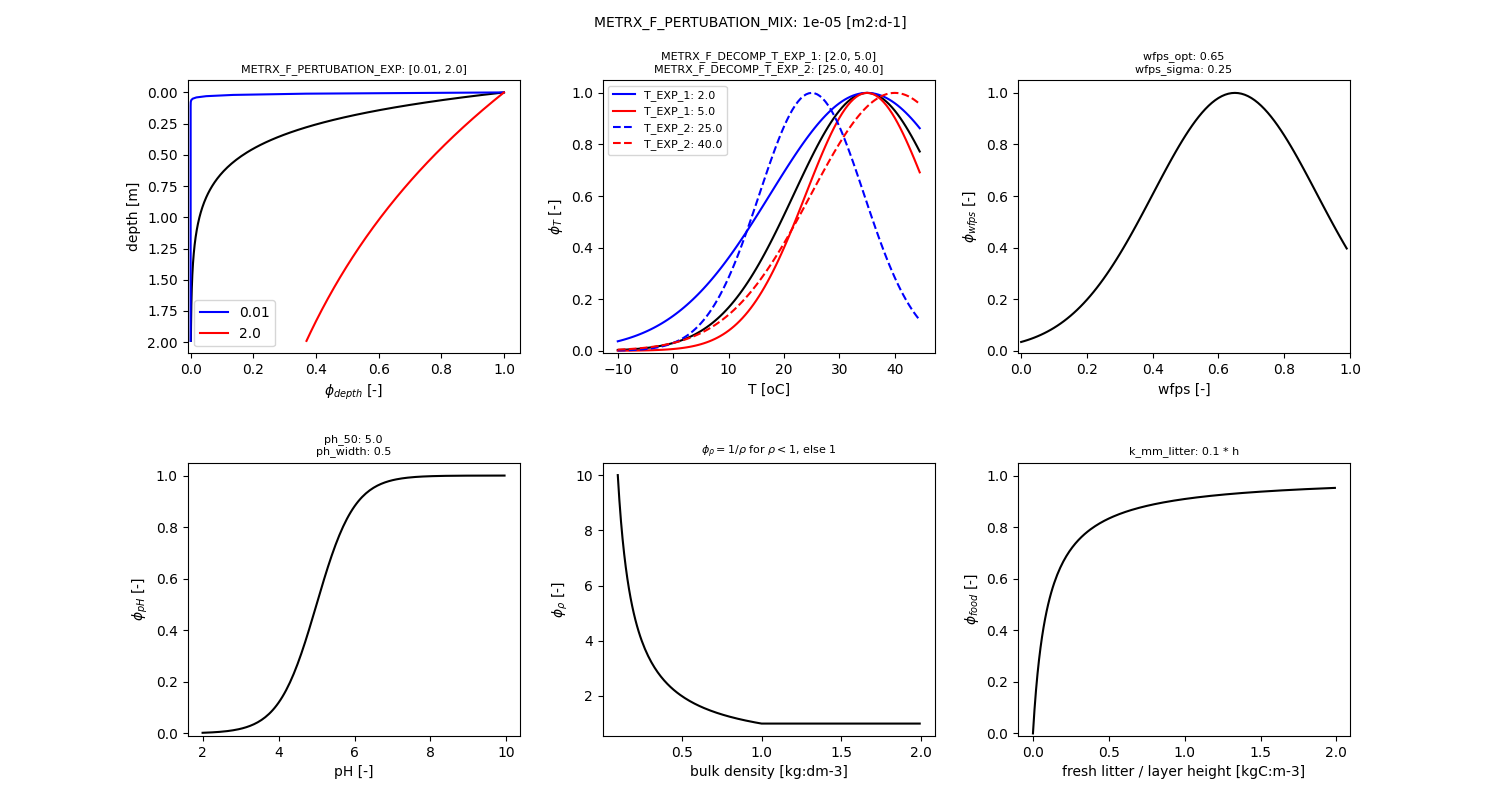
Vertical mixing of soil organic matter due to, e.g., earthworm activity is described as a diffusive process. The effective mixing coefficient \( D_{bio} \) [m2:d-1] of each soil layer is given by a maximum mixing rate that is scaled by several dimensionless response factors:
\[D_{bio} = \Omega_{MIX} \cdot \phi_{z} \cdot \phi_{T} \cdot \phi_{wfps} \cdot \phi_{pH} \cdot \phi_{\rho} \cdot \phi_{food} \]
\[ \phi_{z} = e^{-z / \Omega_{EXP}} \]
\[ \phi_{T} = e^{-\Omega_{T,1} \left(1 - \frac{T}{\Omega_{T,2}}\right)^2} \]
\[ \phi_{wfps} = e^{-\frac{1}{2} \left(\frac{wfps - wfps_{opt}}{\sigma}\right)^2} \]
\[ \phi_{pH} = \frac{1}{1 + e^{-\frac{pH - pH_{50}}{w}}} \]
\[ \phi_{\rho} = \begin{cases} 1 / \rho & \rho < 1 \\ 1 & \rho \geq 1 \end{cases} \]
\[ \phi_{food} = \frac{C_{lit}}{C_{lit} + K_{lit}} \]
Radon (Ra-222) is created via the decay chain of U-238, with Ra-226 as the immediate parent material. It has a half-life of 3.8 days, and during this time can diffuse through the soil and be emitted into the atmosphere. Radon concentration is typically measured in the units Bqm$^{-3}$ - i.e. the number of radon decays per second per cubic metre. LDNDC thus uses the unit Bqm$^{-2}$ for the 'mass' per square metre of Ra-222 in a soil layer. While Bq is a measure of decays per second rathern than mass, it is simple to convert between the two. True mass (kg) can be determined by multiplying by the atomic mass of Ra-222 divided by the Ra-222 decay constant.
Phase equilibrium betwenn dissolved and gaseous state is calculated throughout the soil profile as well as for the top layer of the surface water table (if existing).
For the following species the phase equilibrium betwenn dissolved and gaseousstate is calculated:
For the equilibrium between the partial pressure in the gas pahse \( p_{i,gas} \) and the concentrations in the dissolved species \( i \), the Henry law is applied:
\[ c_{i,liq} = H_{i} p_{i,gas} \]
Gaseous diffusion is calculated for:
For the bottom, a Neuman no-flow boundary condition is used and for the top a Dirichlet boundary condition is used.
Diffusion of dissolved species is calculated for:
The amount of dissolved matter that leaves the simulated domain is added to the leaching output.
If there is a calculated inflow of matter, there is a following correction of mass. The mass is scaled down throughout the whole profile by the amount of calculated mass inflow.
Ebullition is calculated in the soil as well as in the water table. Considered substances are CH4, CO2, O2, NH3, NO, N2O and N2.
Gas bubbles can be fomred as soon as a critical water filled pore space is reached.
Ebullition occurs as soon as total pressure (CH4 + CO2 + ...) exceeds static pressure. Once formed, gas bubbles are transported upwards not being dissolved in upper soil layers as long as water filled pore space is below critical water filled pore space.
If water filled pore space is below critical water filled pore space, gas bubbles are dissolved.
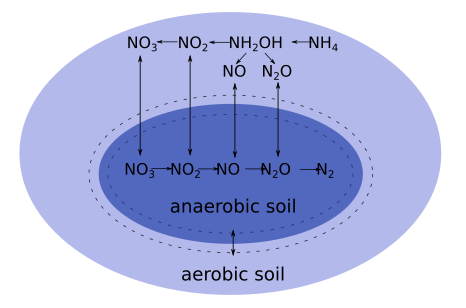
MeTrx considers for a subset of carbon and nitrogen species a horizontal (within one soil layer) differentiation between aerobic and anaerobic parts of the soil. The differentiation is based on the oxygen partial pressure, which in turn is mainly determined by the water profile, respiration processes and gaseous diffusion of oxygen.
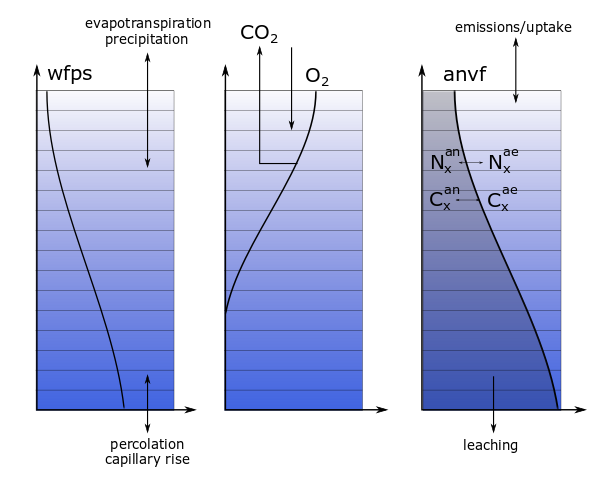
Two anaerobic volumes \( V_{an,x} \) are distinguished, both depending on the oxygen partial pressure \( p_{O_2} \) in bar:
\[ V_{an,r} = e^{-(\Omega_{MFR2} \cdot p_{O_2})^{\Omega_{MFR1}}} \]
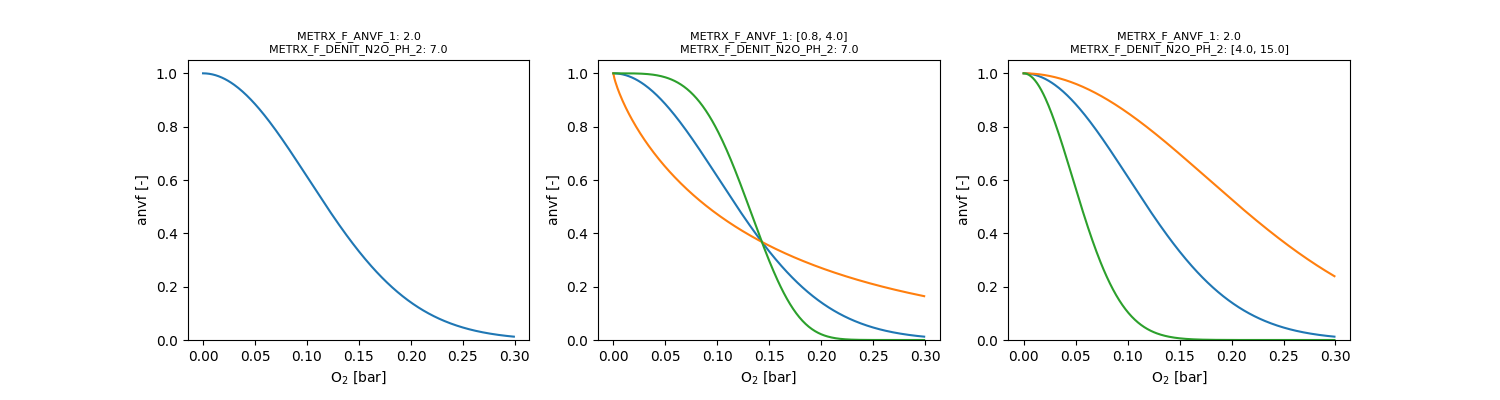
\[ V_{an,s} = e^{-(\Omega_{MFS2} \cdot p_{O_2})^{\Omega_{MFS1}}} \]
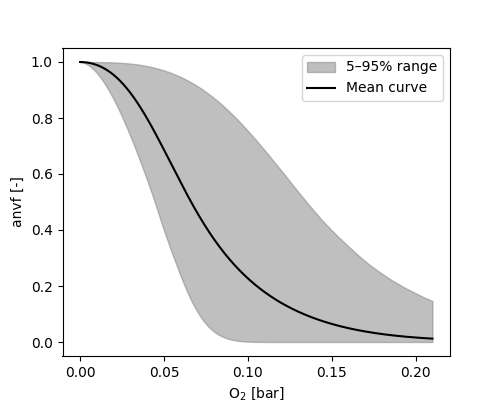
Calibration of both parameters should be restricted to parameter pairs, which yield a response value < 0.2 for partial oxygen pressures at atmospheric conditions.
A change of the size of the anaerobic volume induces redistribution of the aerobic and anerobic part of carbon and nitrogen species.
Redistribution occurs by:
The relative change of a species \( c_x \) only takes place if the share between aerobic and anaerobic volume changes:
\[ \frac{\partial c_{x,an}}{\partial t} = \frac{c_{x,an}}{V_{an}} \frac{\partial V_{an}}{\partial t} \]
\[ \frac{\partial c_{x,ae}}{\partial t} = -\frac{\partial c_{x,an}}{\partial t} \]
The active transport of a species \( c_x \) is given by:
\[ \frac{\partial c_{x,an}}{\partial t} = T^{\ast} \left ( c_{x,an} - c_{x,tot} \frac{V_{an}}{V_{tot}} \right ) \]
\[ \frac{\partial c_{x,ae}}{\partial t} = -\frac{\partial c_{x,an}}{\partial t} \]
The transport coefficient \( T^{\ast} \) is determined by the two parameters:
for gaseous and dissolved species, respectively.
MeTrx considers the following list of synthetic fertilizer:
MeTrx considers the following list of organic fertilizer:
Within the given tilling depth, the following effects are considered:
Urea from fertilizer or manure is dissolved to ammonium in soil and/or in the surface water table depending on temperature:
\begin{eqnarray*}\frac{d NH_4^+}{dT} = N_{urea} \phi_T \\ \frac{d N_{urea}}{dT} = - \frac{d NH_4^+}{dT} \end{eqnarray*}
Depending on the rate of urea hydrolysis, the pH value from of the respective soil layer or water table layer is increased:
\[pH = pH_i + \frac{\frac{d N_{urea}}{dT}}{METRX\_KMM\_PH\_INCREASE\_FROM\_UREA} \]
with \( p_i \) representing the basi pH value that has been defined as model input.
| entity name | decription | unit |
|---|---|---|
| anvf | Anaerobic volume fraction averaged over the complete soil profile | [-] |
| pore_connectivity | Pore connectivity averaged over the complete soil profile | [-] |
| permeability | Permeability averaged over the complete soil profile | [-] |
| wfps | Water filled pore space averaged over the complete soil profile | [-] |
| air | Water filled pore space averaged over the complete soil profile | [-] |
| root_conductivity | Root conductivity averaged over the complete soil profile | [m2s-1] |
| o2 | Sum of oygen mass over the complete soil profile | [kgha-1] |
| t_eff_crnf | ... | [oC] |
| n_release_fraction_crnf | ... | [-] |
| nitrification_inhibition | Inhibition of nitrification | [-] |
| urease_inhibition | Inhibition of urease hydrolysis | [-] |
| carbon_use_efficiency | Carbon use efficiency | [-] |
| N_don | Sum of dissolved organic nitrogen mass over the complete soil profile | [kgha-1] |
| N_nh4 | Sum of ammonium mass over the complete soil profile | [kgha-1] |
| N_nh4_clay | Sum of ammonium adsorbed to clay minerals mass over the complete soil profile | [kgha-1] |
| N_urea | Sum of urea mass over the complete soil profile | [kgha-1] |
| N_no2_ae | Sum of aerobic NO2 mass over the complete soil profile | [kgha-1] |
| N_no2_an | Sum of anaerobic NO2 mass over the complete soil profile | [kgha-1] |
| N_no3_ae | Sum of aerobic NO3 mass over the complete soil profile | [kgha-1] |
| N_no3_an | Sum of anaerobic NO3 mass over the complete soil profile | [kgha-1] |
| N_n2o_ae | Sum of aerobic N2O mass over the complete soil profile | [kgha-1] |
| N_n2o_an | Sum of anaerobic N2O mass over the complete soil profile | [kgha-1] |
| N_no_ae | Sum of aerobic NO mass over the complete soil profile | [kgha-1] |
| N_no_an | Sum of anaerobic NO mass over the complete soil profile | [kgha-1] |
| N_nh3_gas | Sum of gaseous ammonia mass over the complete soil profile | [kgha-1] |
| N_nh3_liq | Sum of dissolved ammonia mass over the complete soil profile | [kgha-1] |
| C_doc_ae | Dissolved organic carbon (aerobic soil volume) | [kgCha-1] |
| C_doc_an | Dissolved organic carbon (anaerobic soil volume) | [kgCha-1] |
| C_acetate | Acetate | [kgCha-1] |
| C_ch4_gas | Methane in gas phase | [kgCha-1] |
| C_ch4_liq | Dissolved methane | [kgCha-1] |
| C_aorg | Amount of carbon in active organic material pool | [kgCha-1] |
| N_aorg | Amount of carbon in active organic material pool | [kgNha-1] |
| C_micro_1 | Amount of carbon in microbial pool 1 | [kgCha-1] |
| C_micro_2 | Amount of carbon in microbial pool 2 | [kgCha-1] |
| C_micro_3 | Amount of carbon in microbial pool 3 | [kgCha-1] |
| N_micro_1 | Amount of nitrogen in microbial pool 1 | [kgNha-1] |
| N_micro_2 | Amount of nitrogen in microbial pool 2 | [kgNha-1] |
| N_micro_3 | Amount of nitrogen in microbial pool 3 | [kgNha-1] |
| C_humus_1 | Amount of carbon in humus pool 1 | [kgCha-1] |
| C_humus_2 | Amount of carbon in humus pool 2 | [kgCha-1] |
| C_humus_3 | Amount of carbon in humus pool 3 | [kgCha-1] |
| N_humus_1 | Amount of nitrogen in humus pool 1 | [kgNha-1] |
| N_humus_2 | Amount of nitrogen in humus pool 2 | [kgNha-1] |
| N_humus_3 | Amount of nitrogen in humus pool 3 | [kgNha-1] |
| C_litter_soil_1 | Amount of carbon in soil litter pool 1 | [kgCha-1] |
| C_litter_soil_2 | Amount of carbon in soil litter pool 2 | [kgCha-1] |
| C_litter_soil_3 | Amount of carbon in soil litter pool 3 | [kgCha-1] |
| N_litter_soil_1 | Amount of nitrogen in soil litter pool 1 | [kgNha-1] |
| N_litter_soil_2 | Amount of nitrogen in soil litter pool 2 | [kgNha-1] |
| N_litter_soil_3 | Amount of nitrogen in soil litter pool 3 | [kgNha-1] |
| C_algae | Amount of carbon in algae pool | [kgCha-1] |
| N_algae | Amount of nitrogen in algae pool | [kgNha-1] |
| C_litter_stubble | Amount of nitrogen in stubble pool | [kgCha-1] |
| N_litter_stubble | Amount of nitrogen in stubble pool | [kgNha-1] |
| C_total | Total soil organic carbon | [kgCha-1] |
| N_total | Total soil organic nitrogen | [kgNha-1] |
| soc_20cm | Soil organic carbon content in the top 20 cm soil horizon | [%] |
| soc_40cm | Soil organic carbon content in the top 40 cm soil horizon | [%] |
| totn_20cm | Total nitrogen content in the top 20 cm soil horizon | [%] |
| totn_40cm | Total nitrogen content in the top 40 cm soil horizon | [%] |
| fe2_tot | ... | [] |
| fe3_tot | ... | [] |
| till_fact | ... | [] |
| freeze_thaw_fact | ... | [] |
| height_litter | Height of the surface litter layer | [m] |
| ph_watertable | ... | [] |
| ph_soil_surface | ... | [] |
| dN_no3_groundwater | ... | [] |
| dN_assi | ... | [] |
| dN_nit_nh4_no2 | ... | [] |
| dN_nit_no2_no3 | ... | [] |
| dN_nit_no2_no | ... | [] |
| dN_nit_no2_n2o | ... | [] |
| dN_denit_no3_no2 | ... | [] |
| dN_denit_no2_no | ... | [] |
| dN_denit_no2_n2o | ... | [] |
| dN_denit_no2_n2 | ... | [] |
| dN_denit_no_n2o | ... | [] |
| dN_denit_no_n2 | ... | [] |
| dN_denit_n2o_n2 | ... | [] |
| dN_chemodenit_no2_no | ... | [] |
| dC_ch4_oxidation | Daily CH4 oxidation | [kgCha-1] |
| dC_ch4_oxidation_la | Daily CH4 oxidation by low affinity microbes | [kgCha-1] |
| dC_ch4_oxidation_ha | Daily CH4 oxidation by high affinity microbes | [kgCha-1] |
| dC_ch4_production_hydrogen | ... | [kgCha-1] |
| dC_ch4_production_acetate | ... | [kgCha-1] |
| dC_floor_ch4_plant_diffusion | ... | [kgCha-1] |
| dC_floor_ch4_soil_diffusion | ... | [kgCha-1] |
| dC_floor_ch4_water_diffusion | ... | [kgCha-1] |
| dC_floor_ch4_bubbling | ... | [kgCha-1] |
| dC_leach_ch4 | ... | [kgCha-1] |
| dO_floor_o2_plant_diffusion | ... | [] |
| dC_litter_above | ... | [kgCha-1] |
| dC_litter_below | ... | [kgCha-1] |
| dC_fix_algae | ... | [kgCha-1] |
| dN_fix_algae | ... | [] |
| dC_decomp_litter | ... | [kg:ha-1] |
| dC_co2_prod_mic_1_growth | ... | [kgCha-1] |
| dC_co2_prod_mic_1_maintenance | ... | [kgCha-1] |
| dC_co2_prod_mic_2 | ... | [kgCha-1] |
| dC_co2_prod_mic_3_acetate_prod | ... | [kgCha-1] |
| dC_co2_prod_mic_3_acetate_cons | ... | [kgCha-1] |
| dC_co2_prod_ch4_prod | ... | [kgCha-1] |
| dC_co2_prod_ch4_cons | ... | [kgCha-1] |
| dH_hydrogen_prod | ... | [] |
| dC_acetate_prod | ... | [kgCha-1] |
| dC_acetate_cons_fe3 | ... | [kgCha-1] |
| dH_hydrogen_cons_fe3 | ... | [] |
| dC_doc_prod_litter | ... | [kgCha-1] |
| dC_doc_prod_humus | ... | [kgCha-1] |
| dC_doc_prod_aorg | ... | [kgCha-1] |
| dC_doc_prod_plant | ... | [kgCha-1] |
| dC_doc_prod_total | ... | [kgCha-1] |
| dC_humify_mic_hum_2 | ... | [kgCha-1] |
| dC_humify_hum_1_hum_2 | ... | [kgCha-1] |
| dC_humify_hum_2_hum_3 | ... | [kgCha-1] |
| entity name | decription | unit |
|---|---|---|
| N_nh4 | Ammonium | [kgNm-2] |
| N_no3 | Nitrate | [kgNm-2] |
| C_doc | Dissolved organic carbon | [kgCm-2] |
| sC_ch4_ebul | CH4 emissions via ebullition | [kgCm-2] |
| sC_ch4_plant | CH4 emissions via plant mediated diffusion | [kgCm-2] |
| sC_ch4_soil | CH4 emissions via soil surface | [kgCm-2] |
| sC_ch4_water | CH4 emissions via surface water table | [kgCm-2] |
| sC_ch4_leach | CH4 leaching | [kgCm-2] |
| sC_ch4_prod | CH4 production | [kgCm-2] |
| sC_ch4_ox | CH4 oxidation | [kgCm-2] |
| sC_acetate_prod | Acetate production | [kgCm-2] |
| sC_doc_prod | DOC production | [kgCm-2] |
| sN_no3_denit | NO3 denitrification | [kgNm-2] |
| sN_n2o_ebul | N2O emissions via ebullition | [kgNm-2] |
| sN_n2o_plant | N2O emissions via plant mediated diffusion | [kgNm-2] |
| sN_n2o_soil | N2O emissions via soil surface | [kgNm-2] |
| sN_n2o_water | N2O emissions via surface water table | [kgNm-2] |
| sN_no_ebul | NO emissions via ebullition | [kgNm-2] |
| sN_no_plant | NO emissions via plant mediated diffusion | [kgNm-2] |
| sN_no_soil | NO emissions via soil surface | [kgNm-2] |
| sN_no_water | NO emissions via surface water table | [kgNm-2] |
| sN_nh3_ebul | NH3 emissions via ebullition | [kgNm-2] |
| sN_nh3_plant | NH3 emissions via plant mediated diffusion | [kgNm-2] |
| sN_nh3_soil | NH3 emissions via soil surface | [kgNm-2] |
| sN_nh3_water | NH3 emissions via surface water table | [kgNm-2] |
| sO_plant_o2_cons | Oxygen consumption by roots | [kgOm-2] |
| sO_plant_o2_prod | Oxygen release by roots | [kgOm-2] |
| sO_algae_o2_prod | Oxygen release by algae | [kgOm-2] |
| ph_watertable | Mean pH value in the surface water table | [-] |
| ph_soil_surface | Mean pH value in the soil | [-] |
| anvf | Anaerobic volume fraction | [%] |
| entity name | decription | unit |
|---|---|---|
| layer | Soil layer | [-] |
| level | Soil layer level (positive from soil surface upwards) | [m] |
| extension | extension | [m] |
| pH | pH value | [-] |
| pore_connectivity | Connectivity of pores | [0-1] |
| relative_permeability | Relative permeability of gaseous diffusion | [0-1] |
| aerenchym_permeability | Aerenchym permeability | [...] |
"cfdd[oC]", water_content | Water content | [0-1] air_content | Air content | [0-1] porosity | Porosity | [0-1] fe2 | Iron Fe2+ [kg:ha-1] fe3 | Iron Fe3+ | [kg:ha-1] C_co2 | CO2 content | [kg:ha-1] C_ch4 | CH4 content | [kg:ha-1] dC_ch4_bubbling | CH4 transport via ebullition | [kg:ha-1] dC_ch4_production | CH4 production | [kg:ha-1] dC_ch4_oxidation | CH4 oxidation | [kg:ha-1] dC_doc_production | DOC production | [kg:ha-1] dC_acetate_production | Acetate production | [kg:ha-1] dC_microbial_death | Microbial death | [kg:ha-1] C_doc | Dissolved organic carbon | [kg:ha-1] C_acetate | Acetate | [kg:ha-1] N_no3 | NO3 | [kg:ha-1] N_nh4 | NH4 | [kg:ha-1] N_urea | IUrea | [kg:ha-1] N_nh3 | NH3 | [kg:ha-1] o2 | Oxygen partial pressure | [bar] N_no | NO content | [kg:ha-1] N_n2o | N2O content | [kg:ha-1] C_humus_1 | Humus pool 1 | [kg:ha-1] C_humus_2 | Humus pool 2 | [kg:ha-1] C_humus_3 | Humus pool 3 | [kg:ha-1] dN_no3_cons_denit | Denitrification of NO3 | [kg:ha-1] denit_factor_c | Factor of denitrification dependency on carbon availability | [0-1] denit_factor_n | Factor of denitrification dependency on nitrogen availability | [0-1] dN_no3_prod_nit | NO3 production from nitrificartion | [kg:ha-1] dN_no3_transport | Downward transport of NO3 | [kg:ha-1]
| entity name | decription | unit |
|---|---|---|
| C_surface | Surface C-litter | [kgCm-2] |
| C_soil_20cm | Total soil carbon in 20 cm topsoil | [kgCm-2] |
| C_humus_1_20cm | Carbon in humus pool 1 in 20 cm topsoil | [kgCm-2] |
| C_humus_2_20cm | Carbon in humus pool 1 in 20 cm topsoil | [kgCm-2] |
| C_humus_3_20cm | Carbon in humus pool 1 in 20 cm topsoil | [kgCm-2] |
| C_litter_20cm | Carbon in litter pools in 20 cm topsoil | [kgCm-2] |
| C_aorg_20cm | Carbon aorg pool in 20 cm topsoil | [kgCm-2] |
Liming raises the base pH of all soil layers starting above the liming depth ("depth", default: 0.3 m) to the target pH ("ph_target"), layers with a higher pH remain unchanged. The base pH is the pH given as model input, which may be temporarily increased, e.g., by urea hydrolysis.
Liming is triggered by lime events (attributes "type", "amount", "depth", "ph_target") or by automatic liming (see model options). Lime events require "ph_target"; calculating the pH change from the lime "amount" and "type" is not yet supported.
During the spinup simulation years, carbon inputs into and fractional losses (decomposition, humification, transport) from the humus, litter and microbial residue (aorg) pools are accumulated for each soil layer and month. The monthly sums of the last 12 months are kept in a moving window. At the end of each month, the flux-weighted equilibrium of each pool is derived from this window:
\[ C^{eq}_x = \frac{\sum_t I_x(t) - \Delta C_x}{\sum_t k_x(t)} \]
with the carbon input \( \sum_t I_x(t) \) and the fractional loss rate \( \sum_t k_x(t) \) summed over the window and the share \( \Delta C_x \) of the prescribed annual change of soil organic carbon (spinupdeltac) scaled to the length of the window. With a complete window, spinupdeltac is thus distributed over the year in proportion to the carbon inputs.
Pools are gradually moved towards their equilibrium by a monthly relaxation factor of 1/3 (reduced in proportion while the window is not yet complete). Since carbon inputs into humus pools mainly originate from microbial necromass, which itself is fed by the decomposition of humus, inputs depend on the pool sizes and the monthly updates iteratively approach the equilibrium.
Total carbon of each soil layer is conserved. Priority is given to the more labile pools: the equilibrium of humus pool 1 is determined first, of humus pool 2 second and humus pool 3 receives the remaining carbon.
 1.13.2