 |
LandscapeDNDC 1.37.0
|
|
LandscapeDNDC 1.37.0
|
This WatercycleDNDC model is taken from the PnET-N-DNDC Model (Li 2000). It calculates daily dynamics of snowcover, soil ice content, potential evaporation and hourly dynamics of rainfall, interception, transpiration, percolation, and runoff.
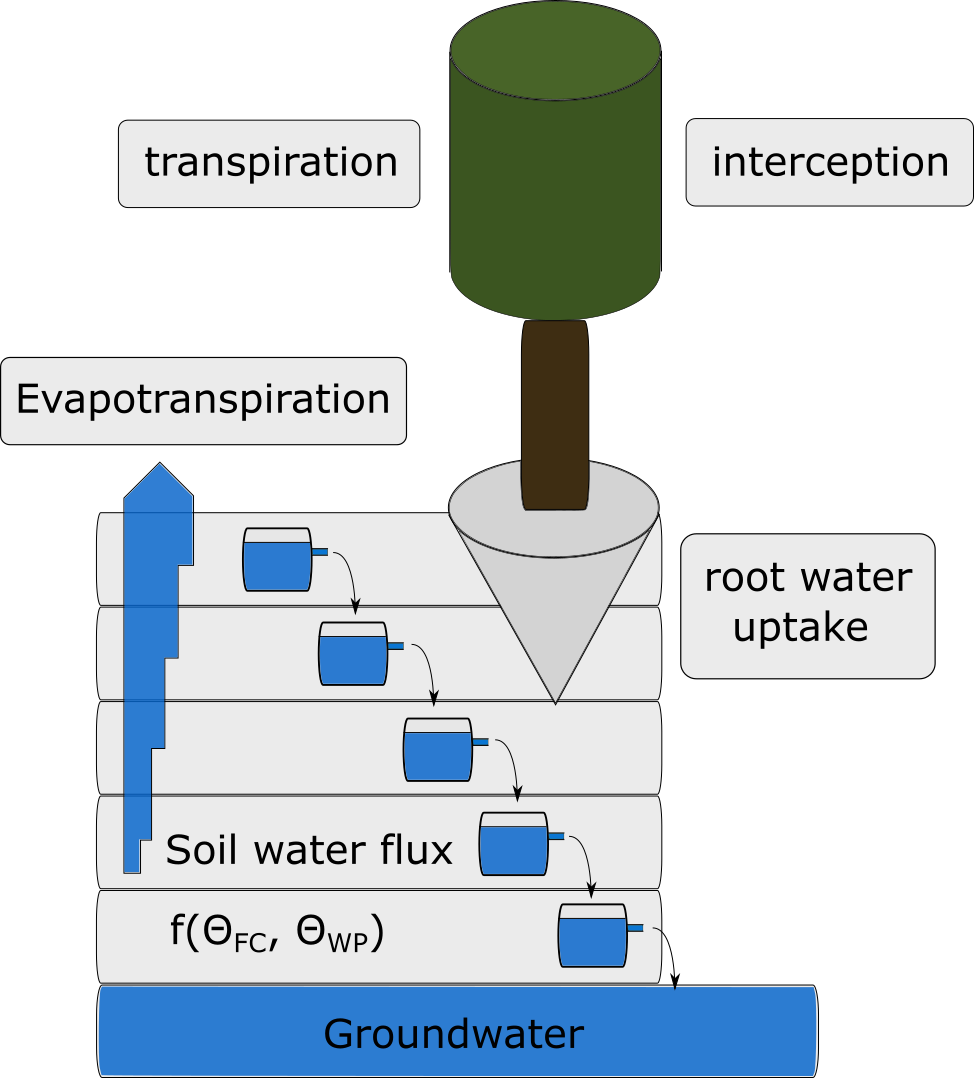
WatercycleDNDC requires further models for:
The following lists include parameters that might be calibrated in order to adapt the model to site conditions:
Interception:
Evapotranspiration:
Preferential flow
Lateral runoff
Percolation
Root water uptake (species parameter)
Available options: Default options are marked with bold letters.
With "potentialevapotranspiration" = penmanmonteith, the wind speed of the climate input is converted to 2 m height if the climate file gives the wind measurement height with the attribute "windheight" [m] (default 2 m; e.g. wind measured on a tower above a forest, see Penman-Monteith (FAO-56)).
\[ wc < wp + x (fc - wp) \]
With the option "evapotranspiration" = previouspattern (default), daily potential evapotranspiration \( PET_d \) is distributed over the time steps of a day following the diurnal course of potential transpiration (calculated by the physiology module) of the last 24 hours. The weights \( w_{ts} \) are updated once per day (first time step of the day):
\[ w_{ts} = \frac{1 - s}{n_{ts}} + s \cdot \frac{T_{ts}}{\sum_{ts} T_{ts}} \]
\[ s = \text{bound}\left(0,\; \frac{T_d}{PET_d},\; 0.9\right) \]
with
The weights sum up to one. Without potential transpiration (e.g., bare soil), \( PET_d \) is distributed uniformly ( \( w_{ts} = 1 / n_{ts} \)). Potential evapotranspiration of a substep is given by \( PET_d \cdot w_{ts} \) divided by the number of substeps per time step.
Actual evapotranspiration is the balance between atmospheric demand of water (potential evapotranspiration) and water supply by the surface. Implemented concepts for the calculation of daily potential evapotranspiration (default: Thornthwaite):
Precipitation of a time step falls with a parameterized rainfall intensity (RI, mm h-1), starting at the beginning of the time step. Thus, the number of hours with rainfall is given by:
\[ n_{rain} = \frac {P}{RI} \]
with
If the precipitation is larger than the rainfall intensity times the number of hours of the time step, rainfall intensity is increased accordingly, i.e., precipitation is evenly distributed over the time step:
\[ ri_{act} = \frac { P }{ n_{hours} } \]
with
The time step is internally subdivided into substeps of substep_hours hours, which receive their respective share of the precipitation of the time step.
Irrigation events are simply added to rainfall.
Selectable flooding regimes via event input:
Both, rainfall and irrigation are subject to interception. The amount of water that can be intercepted depends on:
The interception capacity is defined as the moisture quantity a plant species can harbour on the stems and at the foliage system (see Interception capacity).
All water that is not intercepted feeds into surface water from where it either infiltrates into the soil or is subject to lateral runoff.
Intercepted water contributes to total evapotranspiration. Leaf water evaporation equals the minimum of leaf water and potential evapotranspiration.
Remaining leaf water is redistributed depending on leaf area
Snowfall and soil ice formation are calculated as presented in the library functions Snow and ice .
Update soilwater content due to transpiration.
1) First, the available water for uptake, the fine root density and the inverse capillary pressure are determined for the rooted soil layers. Water can be taken up down to the water content at wilting point:
\[ uptavail_{sl} = (\theta_{sl} - \theta_{wp,sl}) \, h_{sl} \]
The layers are weighted by the composite distribution factor
\[ c_{sl} = uptavail_{sl} \cdot froot_{sl} \cdot \frac{1}{\max(\psi_{sl}, \psi_{fc})} \]
considering available water, fine root distribution (froot) and soil water potential ( \( \psi \), bounded by the potential at field capacity CP_FC).
2) Second, the water uptake target is determined according to the transpiration method of the physiology module:
Note on reference: The 'TREEWATERDEFICIT' option is described in Ziegler et al. (submitted) (will be included when available). This can be used for description, considering that variables and parameters sometimes have slightly different names:
Supply limitation (transpiration methods wateruseefficiency and potentialtranspiration): below a species-specific relative extractable soil water (H2OREF_UPTAKE, 0 = no limitation), the uptake target is reduced linearly (Granier et al. 1999, Ann. For. Sci. 56, 1999: transpiration of temperate forests declines below about 40 % relative extractable water). For each plant, the relative extractable water is weighted by its fine root distribution, and plants are weighted by their fine root mass:
\[ REW_{vt} = \sum_{sl} ffrt_{vt,sl} \, \frac{\theta_{sl} - \theta_{wp,sl}}{\theta_{fc,sl} - \theta_{wp,sl}}, \quad target = target \, \sum_{vt} \frac{m_{frt,vt}}{\sum m_{frt}} \, \min\left(1, \frac{REW_{vt}}{H2OREF\_UPTAKE_{vt}}\right) \]
Without this limitation, uptake continues at the demand rate until the rooted layers reach the wilting point.
3) Third, the uptake target is distributed across the rooted soil layers according to the composite factor. The uptake of a layer is limited by its available water; uptake that cannot be provided by a layer is redistributed to the other layers in proportion to their composite factors (iteratively):
\[ upt_{sl} = \min \left( target_{rest} \, \frac{c_{sl}}{\sum_{avail} c}, \; uptavail_{sl} - upt_{sl} \right) \]
4) Actual transpiration and plant water deficit: without plant water deficit (wateruseefficiency), transpiration equals water uptake. Otherwise, the plant water deficit (only trees) changes by the difference between transpiration and water uptake:
\[ waterdef = waterdef_{old} + transp - \sum\limits upt_{sl} \]
The deficit is limited by the water storage of the living wood, \( wcwood_{pot} = \sum (DSAP\_FRESH / DSAP - 1)(m_{sap} + FCOR \, m_{cor}) \) (DSAP_FRESH and DSAP = density of fresh and oven-dried wood, FCOR = fraction of corewood that contributes to the water supply). If the storage is depleted, transpiration is limited to the water uptake (stomatal closure). The relative water content of the stem water storage is
\[ wc_{rel} = \frac{wcwood_{pot} - waterdef}{wcwood_{pot}} \]
This function is called if ROOT_WATER_UPTAKE_COUVREUR = true (false) and model configuration transpiration = true.
It updates the soil water content regarding the root water uptake for transpiration. The root water uptake is modeled by the Couvreur model (first derived in 3d [23], 1d in [24], in the notation in Ref. [16] for every plant species individually. The potential transpiration is split up for different species by the mass fractions. As species parameters KRSINIT, KCOMPINIT, FRTMASSINIT, and HLEAFCRIT = -16000cm (constant by stomatal regulation) enter.
An effective soil water pressure head ( \( h<0 \) for unsaturated soil, [L][cm]) is determined by
\[h_{eff} = \sum\limits_{sl=0}^{deepest rooted layer} h(sl) \cdot frcfrts(sl) \]
The water potentials are determined via the van-Genuchten parametrisation.
The hydraulic conductivites of the root system \(K_{rs}\) [m/m/h] and for compensation \(K_{comp}\) [m/m/h] scale linearly with the root biomass in respect to the initial root biomass FRTMASSINIT. The parameters for initialisation relate to the same plant stage/time.
\[K_{rs} = KRSINIT \cdot m_{frts} / FRTMASSINIT\\ K_{comp} = KCOMPINIT \cdot m_{frts} / FRTMASSINIT\, . \]
They can be understood as the volumetric fraction of water, which is extracted in an hour.
The root water uptake, as the intensive volumentric water fraction [m/m/timestep], from every layer is calculated by
\[S(sl) = \left( K_{rs} \cdot (h_{eff} - h_{leaf} ) + K_{comp} \cdot (h(sl) - h_{eff}) \right) \cdot \frac{massfrts(sl)/layerwidth}{massallfrts}\, . \]
In contrast to Cai 2017, we therefore use the fine root mass density fractions instead of the normalised root length density.
The potentially used water for transpiration ( \(T_{pot}\)) is provided by another module (physiology). The pressure head of the leaves is derived from the potential transpiration, as long as this value remains above the critical leaf water pressure head HLEAFCRIT.
\[\tilde h_{leaf} = h_{eff} - \frac{T_{Pot}}{K_{rs}} \]
a) If \(\tilde h_{leaf} > HLEAFCRIT\), it is \(h_{leaf} = \tilde h_{leaf}\), then \(T_{act} = T_{pot} \),
b) otherwise \( h_{leaf} = HLEAFCRIT\), then \( T_{act} < T_{pot} \).
The values wcmin and wcmax are not used with this root water uptake model, but the water potentials related to the Van-Genuchten parameters. In contrast, in PlaMox, for the drought stress factor, which enters photosynthesis, wcmin and wcmax are used. Therefore, if the hydraulic conductivity of the root system is unrealisitcally small, or if the Van-Genuchten parameters are not chosen in accordance to wcmin and wcmax, the actual transpiration can be smaller than the potential transpiration without the photosynthesis being affected from this. The Van-Genuchten parameters and wcmin, wcmax should be initialised consistently in the site file.
If the potential evapotranspiration (from CalcPotEvapoTranspiration() and reduced by evaporation from intercepted water, transpiration and evaporation from snow) is not yet zero, and if there is water remaining at the surface, water from this remaining surface water evaporates.
If the potential evapotranspiration is larger than the surface water, all the surface water evaporates.
If the amount of surface water is larger than the potential evapotranspiration, the potential evapotranspiration is reached as the actual evapotranspiration and some surface water still remains.
Snow decrease from evaporation (original in unit: evaporation_of_snow) Since potential evaporation is 0 at freezing temperatures, snow evaporation occurs only for snow that can not melt fast enough If there is more evaporation than can be expected with the sum of gross potential evaporation, hourly foliage evaporation and hourly transpiration, the remaining evaporation is assumes to occur from the snow surface. Snow evaporation is limited to 0.13 mm per day (Granger and Male 1978) and is reported as part of surface water evaporation.
Water from a soil layer evaporates if
Amount of water evaporating from a soil layer \( sl \) :
\[E(sl) = \text{bound}\left(0,\; PET \cdot f_{depth}(sl) \cdot f_{water}(sl),\; \min\left(f_{water}(sl) \cdot \theta(sl) \cdot h(sl),\; PET \right) \right) \]
\[f_{depth}(sl) = \frac{\min\left(h(sl),\; EVALIM - z_{top}(sl)\right)}{EVALIM} \cdot \max\left( 0,\; 1-\frac{\min(EVALIM,\; z_c(sl))}{EVALIM} \right) \]
\[f_{water}(sl) = \text{bound}\left(0,\; \left(\frac{\theta(sl)-\theta_{min}(sl)}{\theta_{fc}(sl)}\right)^{f_{clay}},\; 1\right) \]
\[f_{clay} = 1+ SLOPE\_CLAYF \cdot \min\left(1- \frac{fc_{org}(sl)}{CCORG},\; clay(sl)\right) \]
Comments:
Water inflow is limited by either potential inflow, which is either surface inflow or the outflow of the respective overlying soil layers, and inflow capacity.
For soil layers lying within the groundwater table, water flow out of the layer equals water inflow. In this way, soil water is discharged with groundwater with the percolation flow rate of the soil layer above the groundwater table.
If the last soil layer is above the groundwater, water flow out of the domain is given by:
Calculation of water flow ouf of soil layer is distinguished for different water contents:
Water flow from layer \(sl\) to the layer \(sl+1\) below:
\[q = \min\left( \left(1-\frac{\theta_{fc}(sl)}{(\theta(sl) + \theta_{ice}(sl)) \cdot s}\right)^2 \cdot \theta(sl) \cdot h(sl) \cdot f_{sl} \cdot f_{tt} \cdot f_{imp},\; q_{sat} \right) \]
Water flow from layer \(sl\) to the layer \(sl+1\) below (negative values indicate upward flow):
\[q = \left(\frac{\theta(sl)}{\theta_{fc}(sl)} - \frac{\theta(sl+1)}{\theta_{fc}(sl+1)} \right) \cdot \theta(sl) \cdot h(sl) \cdot f_{sl} \cdot f_{tt} \cdot f_{imp} \]
with \( f_{sl}, f_{tt}, f_{imp} \) as defined in Water flow above field capacity
Similar to WaterFlowBelowFieldCapacity but restricts water flow by water availability from soil layer below
Returns saturated water flow per time step accounting for impedance
...
Percolating water is delayed by an impedance factor, which considers the formation of ice lenses in (partially) frozen soil [Lundin (1990), Hansson et al. (2004).] The impedence factor depends on the parameter IMPEDANCE_PAR = 0.
The surface flux gives the water, which runs off horizontally. This only happens if more water than stopped by the bunding (bund height is set in flooding events) is present.
If the bund height == 0:
The fraction of water that has not infiltrated the soil immediatly and is running off from surface water is determined by the site parameter FRUNOFF.
 1.13.2